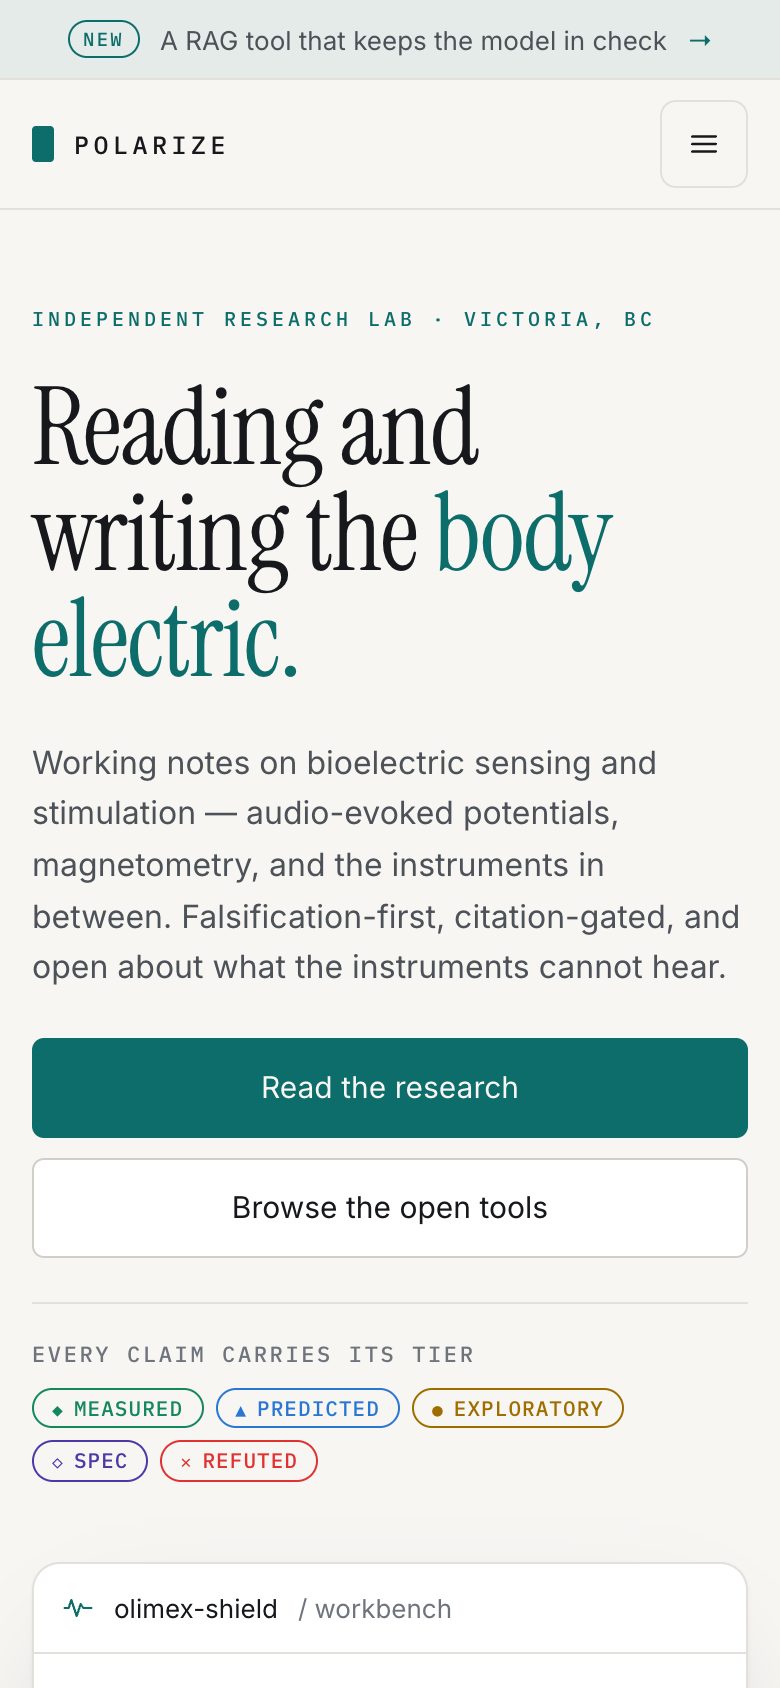
<?xml version="1.0" encoding="utf-8"?><feed xmlns="http://www.w3.org/2005/Atom" ><generator uri="https://jekyllrb.com/" version="3.10.0">Jekyll</generator><link href="https://polarize.tech/blog/feed.xml" rel="self" type="application/atom+xml" /><link href="https://polarize.tech/" rel="alternate" type="text/html" /><updated>2026-10-07T11:10:36-06:00</updated><id>https://polarize.tech/blog/feed.xml</id><title type="html">POLARIZE</title><subtitle>Research notes on audio-evoked potentials, bioelectricity, neuroscience and neuromedicine. Falsification-first, citation-gated.</subtitle><author><name>Joshua Anderton</name></author><entry><title type="html">Redesigning the homepage, one version at a time</title><link href="https://polarize.tech/blog/redesigning-the-homepage/" rel="alternate" type="text/html" title="Redesigning the homepage, one version at a time" /><published>2026-09-28T10:00:00-06:00</published><updated>2026-09-28T10:00:00-06:00</updated><id>https://polarize.tech/blog/redesigning-the-homepage</id><content type="html" xml:base="https://polarize.tech/blog/redesigning-the-homepage/"><![CDATA[<p>Until this week the homepage was a list. It showed the four latest posts, the speculations and
the most recently active repositories, inside the same sidebar layout as every other page. It
was accurate, and it said nothing about what this lab is for.</p>

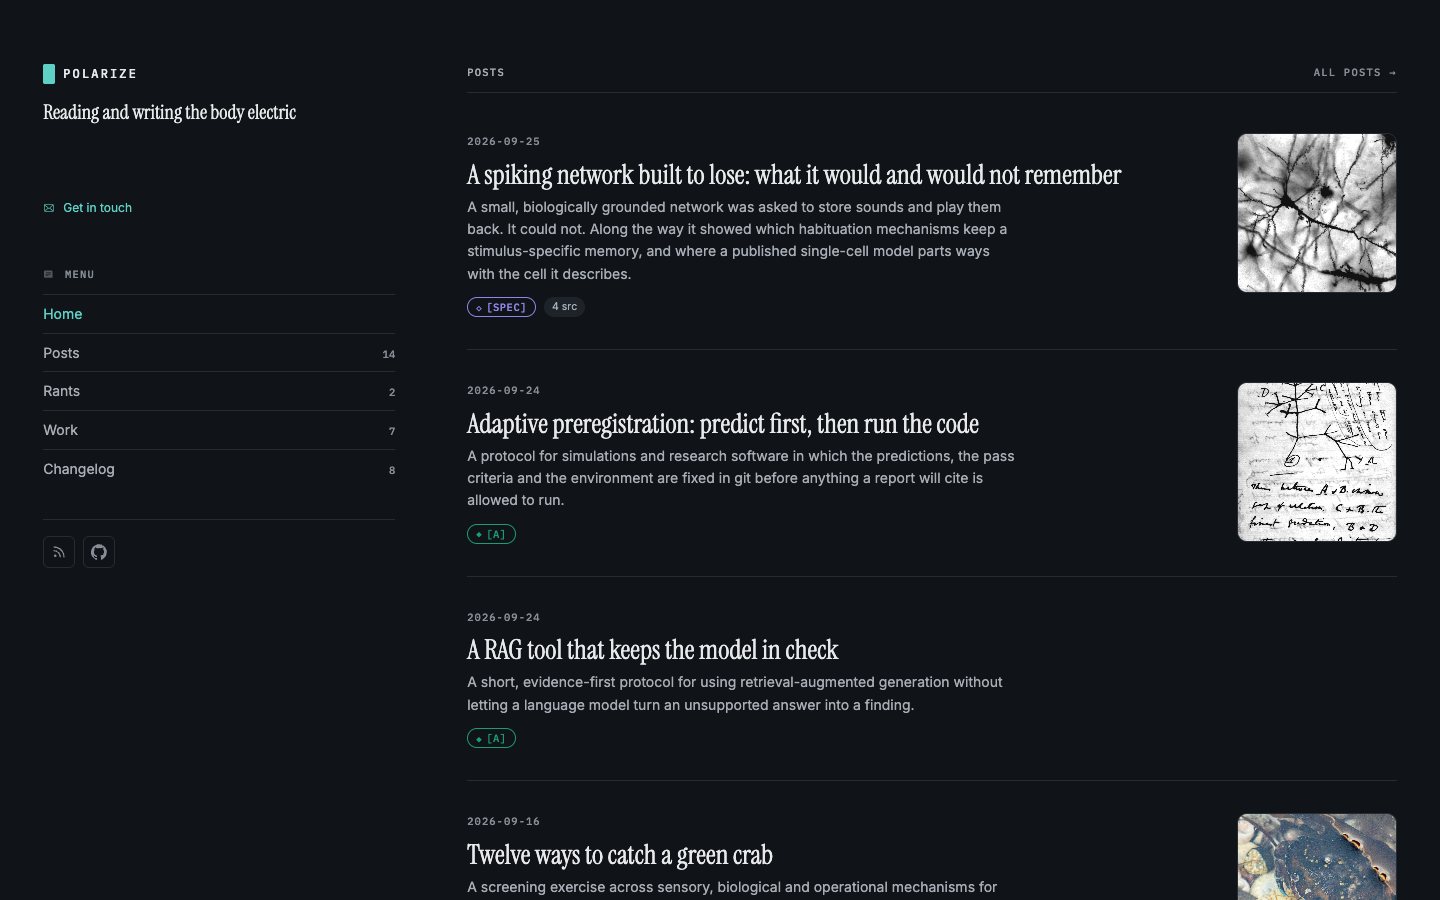
<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/00-before.jpg"><img src="/assets/posts/homepage-redesign/00-before.jpg" alt="The old homepage: a sidebar with the brand, a menu and counts, beside a list of the latest posts with thumbnails." loading="lazy" /></a>
  <figcaption>Before: the homepage as a post list inside the blog's sidebar layout.</figcaption>
</figure>

<p>The redesign was done in the open, in conversation with Claude on a design canvas where every
version stayed side by side. Then it was built with Claude Code. Six directions, oldest first, and then fourteen passes on the last one:</p>

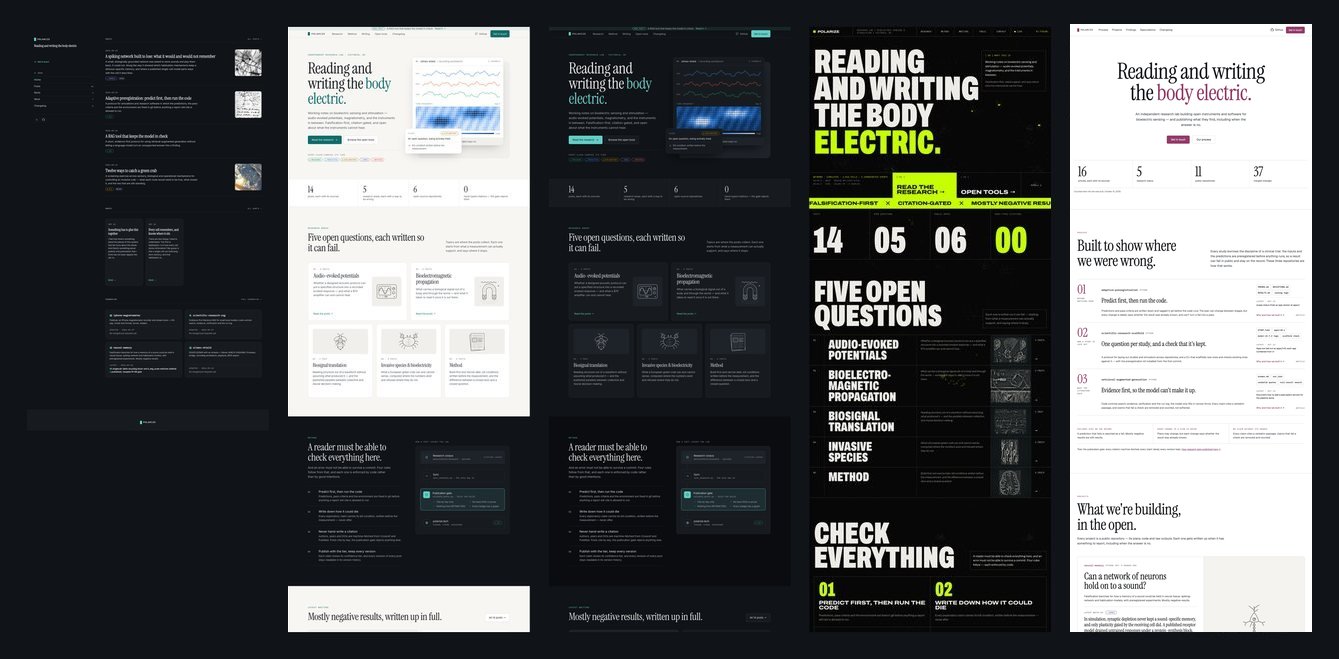
<figure class="shot shot--strip">
  <div class="shot__scroll"><a href="/assets/posts/homepage-redesign/07-filmstrip.jpg"><img src="/assets/posts/homepage-redesign/07-filmstrip.jpg" alt="The top of every homepage version side by side: the old post list, the light version, the dark version, the brutalist version, the no-rules version and the final hybrid." loading="lazy" /></a></div>
  <figcaption>The top of each version, oldest first: before, light, dark, brutalist, no rules, and the one that shipped. Scroll sideways on a phone.</figcaption>
</figure>

<h2 id="1-a-familiar-front-door">1. A familiar front door</h2>

<p>The first brief was a proper homepage for a research lab, borrowing the feel of product sites
like <a href="https://www.digitalocean.com">DigitalOcean</a> and <a href="https://www.intercom.com">Intercom</a>:
a big headline, a product shot, and sections for what the lab does. It was built strictly on
<a href="https://github.com/polarizetech/polarize-ui">polarize-ui</a>, the design system these pages
already used: the display serif for headings, the mono face for labels, and never bold.</p>

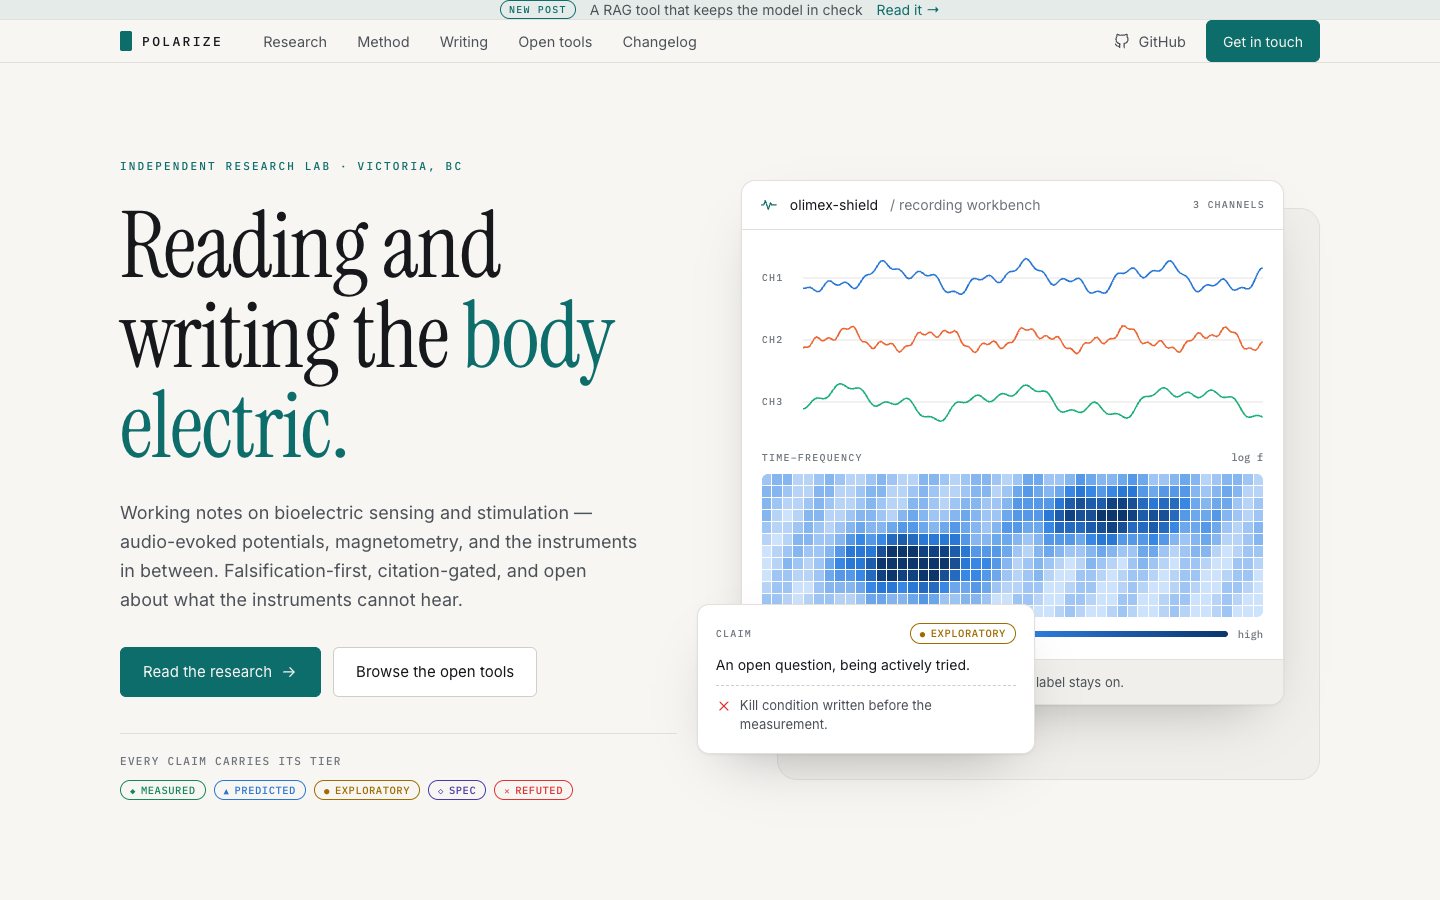
<p>The product shot was a mock recording workbench, with three channels and a time–frequency map.
It carried a TASTE badge saying it was an illustration and not a recording. Even as decoration,
the page kept the rule every page here follows: a label may never be hidden.</p>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/01-light.jpg"><img src="/assets/posts/homepage-redesign/01-light.jpg" alt="Version one: a light page, the heading on the left, a card of waveforms and a heatmap on the right, a claim card overlapping it." loading="lazy" /></a>
  <figcaption>Version one: light, conventional, and entirely inside the design system's rules.</figcaption>
</figure>

<h2 id="2-dark">2. Dark</h2>

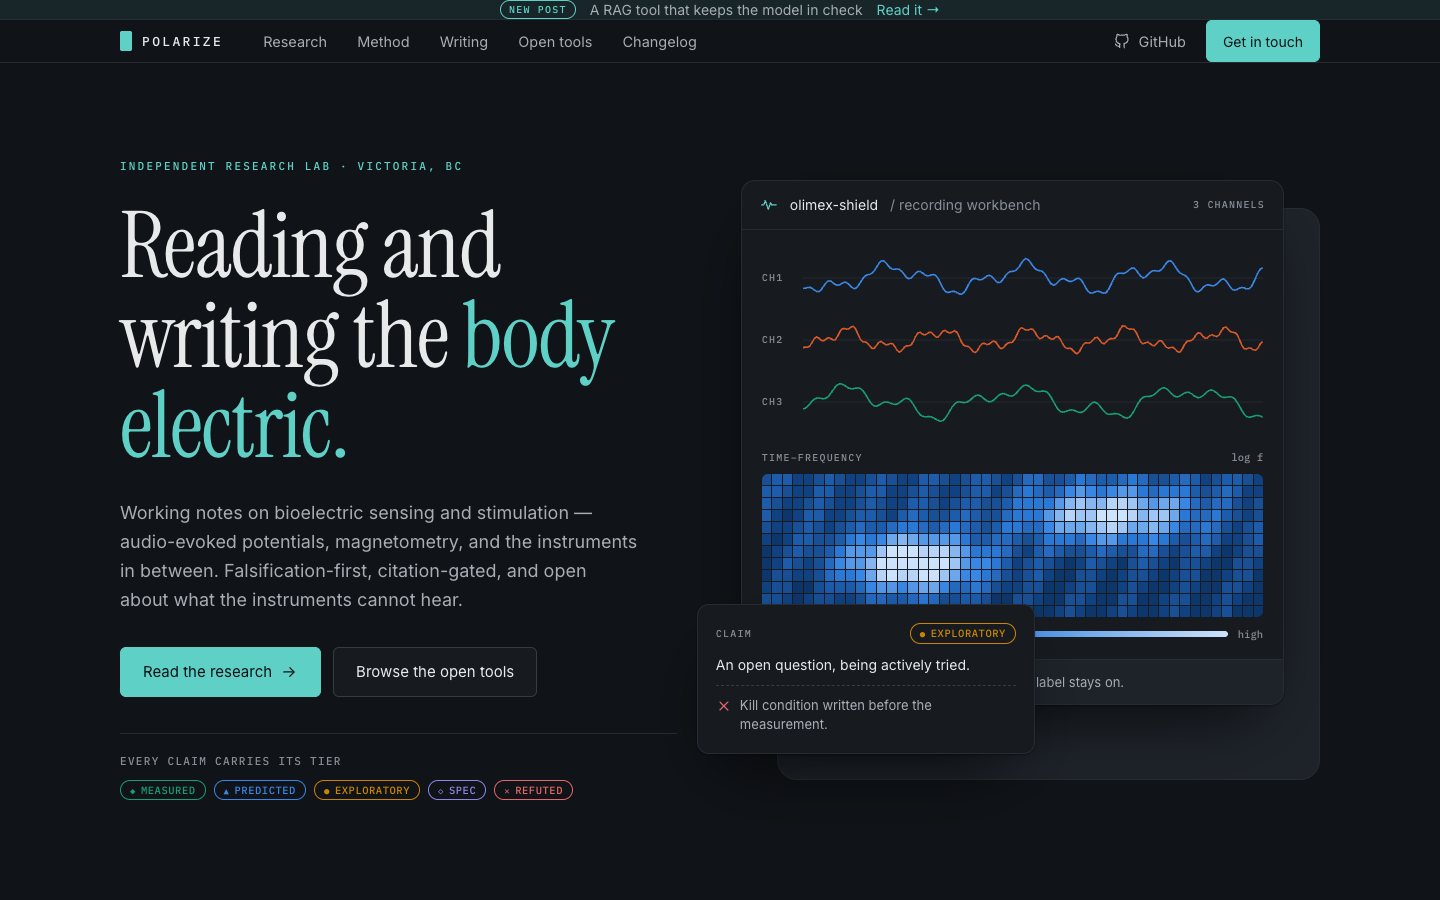
<p>The same page in the design system’s dark palette. It was an easy change, because every colour
is a token. It was also the first sign that the lab reads better at night.</p>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/02-dark.jpg"><img src="/assets/posts/homepage-redesign/02-dark.jpg" alt="Version two: the same layout in a dark palette with a teal accent." loading="lazy" /></a>
  <figcaption>Version two: the same page, dark.</figcaption>
</figure>

<p>Both of the first two versions had a phone layout too, drawn as separate artboards.</p>

<figure class="shot shot--pair">
  <a href="/assets/posts/homepage-redesign/01-light-mobile.jpg"><img src="/assets/posts/homepage-redesign/01-light-mobile.jpg" alt="Version one on a phone: the light page, headline stacked above a smaller waveform card." loading="lazy" /></a>
  <a href="/assets/posts/homepage-redesign/02-dark-mobile.jpg"><img src="/assets/posts/homepage-redesign/02-dark-mobile.jpg" alt="Version two on a phone: the same stacked layout in the dark palette." loading="lazy" /></a>
  <figcaption>Versions one and two at phone width.</figcaption>
</figure>

<h2 id="3-brutalism-and-specks">3. Brutalism, and specks</h2>

<p>Next came a push towards brutalism, after the sound-therapy site <a href="https://byotone.com">Byotōne</a>:
fields of animated specks, bracketed mono tags, a huge headline, and a lettered step-through
navigation. The specks took several forms: a ring around the headline, a slowly turning cell, a
helix, and an evoked-response wave. The page labelled them decoration, not data.</p>

<p>One thing from the reference was deliberately not copied: its all-caps serif. Here uppercase is
always the mono face, so the big headings stayed in regular case.</p>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/03-brutalist.jpg"><img src="/assets/posts/homepage-redesign/03-brutalist.jpg" alt="Version three: a dark page with a ring of specks around a spread-out serif headline, bracketed frequency-band tags and a lettered step navigation." loading="lazy" /></a>
  <figcaption>Version three: specks, bracketed tags, and a stepper that did not survive.</figcaption>
</figure>

<h2 id="4-no-rules">4. No rules</h2>

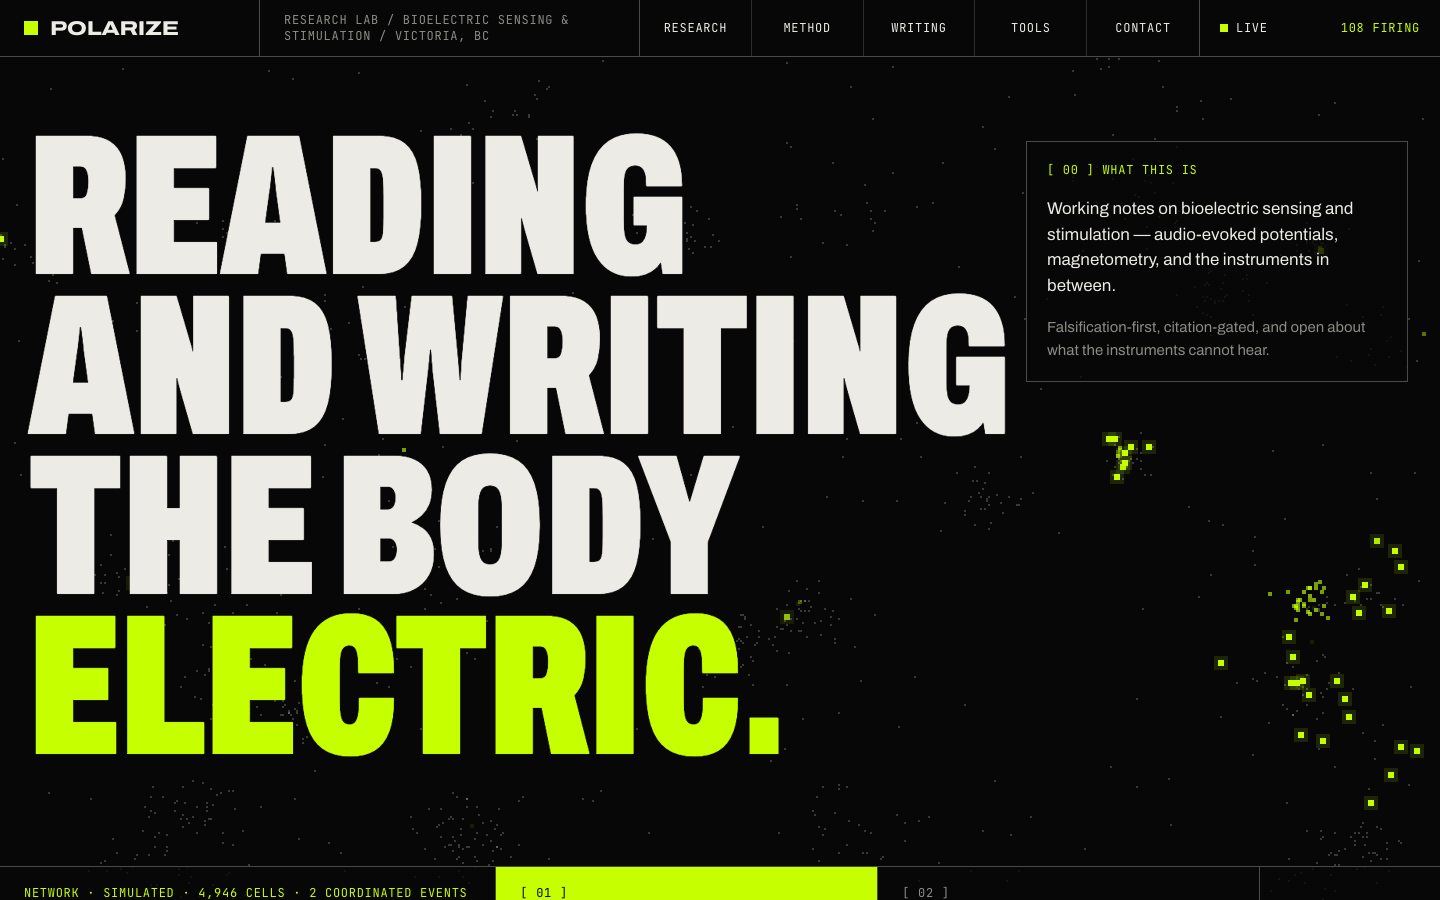
<p>To see what the rules were costing, one version dropped all of them: a condensed grotesque, acid
green, 1px grid lines everywhere, and a simulated network of about five thousand cells behind the
whole page. Those cells fire on their own, set off their neighbours, and sometimes fire together
as waves, synchronised colonies or rhythmic bursts. A live counter in the top bar says how many
are firing, and the footer says it is a simulation.</p>

<p>It was the loudest version and the least like the lab, but the cells stayed.</p>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/04-no-rules.jpg"><img src="/assets/posts/homepage-redesign/04-no-rules.jpg" alt="Version four: an enormous condensed uppercase headline in white and acid green, a grid of mono labels, and clusters of green squares firing in the background." loading="lazy" /></a>
  <figcaption>Version four: no rules. The top bar counts how many simulated cells are firing.</figcaption>
</figure>

<h2 id="5-the-one-that-shipped">5. The one that shipped</h2>

<p>The final version took something from each of the others. It has the dark palette and the design
system’s type. From brutalism it took hard rules and square-ish corners, and from the first
version it took the charts. The cells moved into a single WebGL field behind the entire page, one
that looks like cells polarising rather than confetti. They are small, white, dim, sometimes
grouped, occasionally firing together. The stepper and the bracketed tags went, and so did the
background fills on cards.</p>

<p>The content changed more than the look. Looking at how other labs present themselves helped,
especially <a href="https://drmichaellevin.org">Michael Levin’s lab site</a> and his separate essay site,
<a href="https://thoughtforms.life">Thoughtforms</a>. They pointed to an order: lead with the work, let the
articles report what it found, and give speculation its own quieter room. So the homepage now opens
with the process that keeps results honest. Then come the projects, the changelog, the findings,
the speculations and the design system.</p>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/05-hybrid.jpg"><img src="/assets/posts/homepage-redesign/05-hybrid.jpg" alt="Version five on the canvas: the centred serif headline over a field of faint white specks." loading="lazy" /></a>
  <figcaption>The shipped design, as it stood on the canvas.</figcaption>
</figure>

<h3 id="fourteen-passes-on-the-hybrid">Fourteen passes on the hybrid</h3>

<p>The hybrid itself changed fourteen times before it shipped, one request at a time. These are all
of them, in order, each shown where it changed the page.</p>

<div class="shot-grid">
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h01-hero.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h01-hero.jpg" alt="Step 5.1 of the hybrid homepage: The first hybrid: brutalism's dark palette and specks, the first version's charts, and no stepper." loading="lazy" /></a>
    <figcaption><strong>5.1</strong> · The first hybrid: brutalism's dark palette and specks, the first version's charts, and no stepper.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h02-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h02-focus.jpg" alt="Step 5.2 of the hybrid homepage: Corners down to 4px." loading="lazy" /></a>
    <figcaption><strong>5.2</strong> · Corners down to 4px.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h03-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h03-focus.jpg" alt="Step 5.3 of the hybrid homepage: The specimen drawings replaced by the archival plates the site already had." loading="lazy" /></a>
    <figcaption><strong>5.3</strong> · The specimen drawings replaced by the archival plates the site already had.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h04-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h04-focus.jpg" alt="Step 5.4 of the hybrid homepage: Background fills taken off the cards." loading="lazy" /></a>
    <figcaption><strong>5.4</strong> · Background fills taken off the cards.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h05-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h05-focus.jpg" alt="Step 5.5 of the hybrid homepage: Rebuilt around the repositories: projects first, then the changelog, findings and notes." loading="lazy" /></a>
    <figcaption><strong>5.5</strong> · Rebuilt around the repositories: projects first, then the changelog, findings and notes.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h06-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h06-focus.jpg" alt="Step 5.6 of the hybrid homepage: “Merged this week” became “Recently merged”." loading="lazy" /></a>
    <figcaption><strong>5.6</strong> · “Merged this week” became “Recently merged”.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h07-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h07-focus.jpg" alt="Step 5.7 of the hybrid homepage: One WebGL field behind the whole page. At first the cells looked like bubbles." loading="lazy" /></a>
    <figcaption><strong>5.7</strong> · One WebGL field behind the whole page. At first the cells looked like bubbles.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h08-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h08-focus.jpg" alt="Step 5.8 of the hybrid homepage: Back to specks: smaller, clustered, of varying density." loading="lazy" /></a>
    <figcaption><strong>5.8</strong> · Back to specks: smaller, clustered, of varying density.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h09-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h09-focus.jpg" alt="Step 5.9 of the hybrid homepage: One colour: a faded white that polarises in opacity only." loading="lazy" /></a>
    <figcaption><strong>5.9</strong> · One colour: a faded white that polarises in opacity only.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h10-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h10-focus.jpg" alt="Step 5.10 of the hybrid homepage: Quieter still: lower peaks, softer firing." loading="lazy" /></a>
    <figcaption><strong>5.10</strong> · Quieter still: lower peaks, softer firing.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h11-hero.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h11-hero.jpg" alt="Step 5.11 of the hybrid homepage: The bracketed corner tags removed." loading="lazy" /></a>
    <figcaption><strong>5.11</strong> · The bracketed corner tags removed.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h12-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h12-focus.jpg" alt="Step 5.12 of the hybrid homepage: A Process section: three repositories that keep results honest." loading="lazy" /></a>
    <figcaption><strong>5.12</strong> · A Process section: three repositories that keep results honest.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h13-hero.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h13-hero.jpg" alt="Step 5.13 of the hybrid homepage: A simpler, centred hero; the numbers strip gone." loading="lazy" /></a>
    <figcaption><strong>5.13</strong> · A simpler, centred hero; the numbers strip gone.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h13-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h13-focus.jpg" alt="Step 5.13 of the hybrid homepage: The charts moved into a section for polarize-ui." loading="lazy" /></a>
    <figcaption><strong>5.13</strong> · The charts moved into a section for polarize-ui.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h14-hero.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h14-hero.jpg" alt="Step 5.14 of the hybrid homepage: A dedicated cell turning behind the heading, with buttons for the process and for getting in touch." loading="lazy" /></a>
    <figcaption><strong>5.14</strong> · A dedicated cell turning behind the heading, with buttons for the process and for getting in touch.</figcaption>
  </figure>
  <figure class="shot">
    <a href="/assets/posts/homepage-redesign/hybrid/h14-focus.jpg"><img src="/assets/posts/homepage-redesign/hybrid/h14-focus.jpg" alt="Step 5.14 of the hybrid homepage: Speculations as story cards, told like posts." loading="lazy" /></a>
    <figcaption><strong>5.14</strong> · Speculations as story cards, told like posts.</figcaption>
  </figure>
</div>

<h2 id="6-from-canvas-to-components">6. From canvas to components</h2>

<p>A design that lives only on a canvas has to be rebuilt by hand for every page, and it drifts. So
it went into polarize-ui as components, in both of its forms: a zero-build stylesheet and custom
element for plain HTML sites like this one, and React components that render the same classes.</p>

<p>The new landing layer covers the top bar, hero, section heads, process steps, project features,
repository cards, the changelog feed, article cards, story cards, archival plates and the footer.
The cell field is <code class="language-plaintext highlighter-rouge">&lt;ui-cellfield&gt;</code>. It draws nothing a reader needs, and it stops for anyone who
has asked their system to reduce motion. The design system’s own checks hold the new stylesheet
to the same rules as the rest: no raw colours, never bold, and uppercase only in the mono face.</p>

<p>It shipped as polarize-ui v0.5.6, and this site then adopted it everywhere. Every page now has the
new top bar, the new footer and the dark palette, and the speculations page uses the new story
cards.</p>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/06-live-process.jpg"><img src="/assets/posts/homepage-redesign/06-live-process.jpg" alt="The live Process section: three numbered cards for adaptive-preregistration, scientific-research-scaffold and scientific-research-rag, joined by arrows." loading="lazy" /></a>
  <figcaption>Live: the Process section, three repositories that keep results honest.</figcaption>
</figure>

<figure class="shot shot--wide">
  <a href="/assets/posts/homepage-redesign/06-live-findings.jpg"><img src="/assets/posts/homepage-redesign/06-live-findings.jpg" alt="The live Findings section: a featured article with its photograph beside its title and summary." loading="lazy" /></a>
  <figcaption>Live: Findings, built from the posts themselves, with their own images and credits.</figcaption>
</figure>

<p>The same components hold up on a phone. The top bar folds into a menu that works without script,
the process steps stack with downward arrows, and the story cards scroll sideways.</p>

<figure class="shot shot--pair">
  <a href="/assets/posts/homepage-redesign/06-live-mobile.jpg"><img src="/assets/posts/homepage-redesign/06-live-mobile.jpg" alt="The live homepage on a phone: the heading, description and two buttons over the cell field." loading="lazy" /></a>
  <a href="/assets/posts/homepage-redesign/06-live-mobile-process.jpg"><img src="/assets/posts/homepage-redesign/06-live-mobile-process.jpg" alt="The Process section on a phone: one numbered card per row." loading="lazy" /></a>
  <figcaption>On a phone: the hero, and the process steps stacked.</figcaption>
</figure>

<h2 id="what-was-kept">What was kept</h2>

<p>Every version is still on the canvas, and the rules did most of the work. The versions that broke
them were useful for finding out what the rules cost, and each time the answer was less than it
first looked. These are the ones that survived:</p>

<ul>
  <li><strong>The type rules.</strong> The display serif is for headings, the sans is never bold, and uppercase is
always mono.</li>
  <li><strong>The label rule.</strong> Decoration says it is decoration. A tier badge can never be hidden.</li>
  <li><strong>Real content only.</strong> Every card is built from the site’s own data: posts, essays, repositories
and the changelog. A project’s finding is always its own post’s summary, never a line written for
the homepage.</li>
  <li><strong>The cells.</strong> Only these came from the version with no rules.</li>
</ul>

<p>The components are in <a href="https://github.com/polarizetech/polarize-ui">polarize-ui</a>, and the live
Storybook shows the whole homepage at desktop and phone width.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[Six versions of the polarize.tech homepage, from a post list in a sidebar to a lab's front door drawn over a field of polarising cells: what each one tried, what was kept, and how the result became components in the design system.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/homepage-redesign.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/homepage-redesign.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">One question per study: laying out research across repositories</title><link href="https://polarize.tech/blog/one-question-per-study/" rel="alternate" type="text/html" title="One question per study: laying out research across repositories" /><published>2026-09-28T09:00:00-06:00</published><updated>2026-09-28T09:00:00-06:00</updated><id>https://polarize.tech/blog/one-question-per-study</id><content type="html" xml:base="https://polarize.tech/blog/one-question-per-study/"><![CDATA[<p>Preregistration decides the order things happen in inside one experiment. It says nothing about
where the experiment lives. The work here is spread across repositories: a bench in one, a
simulator in another, shared tools in a monorepo, and findings in a separate research corpus.
The layout was being decided one repository at a time, and a decision made that way is a
decision nobody checks.</p>

<p><a href="https://github.com/polarizetech/scientific-research-scaffold">scientific-research-scaffold</a>
is the result of writing those decisions down once. It is a protocol for how a piece of research
is laid out across repositories, and <code class="language-plaintext highlighter-rouge">scaffold</code>, a small command-line tool that sets new
repositories up in that shape and checks existing ones against it.</p>

<h2 id="what-the-layout-has-to-protect">What the layout has to protect</h2>

<p>Every rule in the protocol exists to keep a result checkable by someone who is not the author,
on a machine that is not the author’s. Four things break that quietly:</p>

<ul>
  <li><strong>A classification baked into a name.</strong> A simulator here started life as <code class="language-plaintext highlighter-rouge">sim-neural-memory</code>
and was later renamed to <code class="language-plaintext highlighter-rouge">neural-memory</code>. A prefix fixes a category into a name that outlives
it, and renaming breaks every link and path that pointed at the old one.</li>
  <li><strong>Two copies of one thing.</strong> A simulator imported as a folder by two studies is two copies
waiting to diverge.</li>
  <li><strong>A path on one person’s machine.</strong> A result produced through an absolute home-directory path
is a result nobody else can regenerate.</li>
  <li><strong>Findings in more than one place.</strong> A research corpus mounted inside each study is several
working copies of one record, and they drift.</li>
</ul>

<h2 id="two-kinds-of-repository">Two kinds of repository</h2>

<p>The protocol has two kinds of repository, declared in a manifest rather than in the name:</p>

<ul>
  <li>A <strong>study</strong> is one research question and everything used to pursue it: small versioned apps
for exploring it by hand, simulators for modelling it, preregistered experiments for testing
it, and pinned datasets to test it against.</li>
  <li>A <strong>sim</strong> is one simulator under adaptive preregistration. Its versions are tags inside one
repository, never new repositories.</li>
</ul>

<p>Neither holds findings. A study’s findings go to the shared corpus, and the study refers to them
by claim ID. Everything specific to one organisation (which repository is the corpus, which design
system the apps use, where shared tools live) sits in a profile, so the protocol itself stays
generic and can be forked.</p>

<p>An app is for exploring and an experiment is for testing. An app answers “is this worth testing?”
A number from an app is never a finding; a finding comes from a preregistered experiment.</p>

<h2 id="when-a-simulator-moves-out">When a simulator moves out</h2>

<p>A simulator starts as a folder inside the study that needs it. It moves to its own repository when
one of three things becomes true: a second study uses it, it needs releases on its own schedule,
or it is shared outside on its own. Tidiness, size and “it might be reused someday” are not
reasons.</p>

<p><code class="language-plaintext highlighter-rouge">scaffold promote-sim</code> does the mechanical part. It splits the folder’s history into its own
branch, so the new repository keeps every commit, and the study then pins the new repository by
tag like any other dependency.</p>

<h2 id="strictness-that-scales-and-rules-that-dont">Strictness that scales, and rules that don’t</h2>

<p>How strict a repository has to be depends on what a mistake would cost, and the protocol names
four stages. A sketch owes honest labels and a note of what was not done. Once a number is being
produced, it owes a preregistration before any run that could be quoted. Once another repository
depends on it, or a number from it is quoted, it owes CI, a lockfile and tagged releases. Once
someone outside relies on it, it owes a frozen release, a DOI and an external preregistration.</p>

<p>Some things never relax at any stage: the safety of anyone taking part, honest labels, other
people’s data licences, and saying plainly what was not done.</p>

<h2 id="what-the-tool-does">What the tool does</h2>

<p><code class="language-plaintext highlighter-rouge">scaffold new study</code> renders a template, makes the first commit, installs the
<a href="https://github.com/polarizetech/adaptive-preregistration">preregistration kit</a>, and prints the
command that would create the repository on GitHub. It leaves the visibility decision to the
person, and it never publishes anything. <code class="language-plaintext highlighter-rouge">scaffold new app</code> adds the next versioned app, and
<code class="language-plaintext highlighter-rouge">scaffold new sim</code> adds a simulator, inside a study or as its own repository.</p>

<p><code class="language-plaintext highlighter-rouge">scaffold check</code> is the part that matters day to day. It confirms that the manifest is valid,
that the name carries no prefix, and that the kind in the README matches the manifest. It checks
that visibility was decided and dated, that the preregistration kit is installed, and that every
external simulator is pinned to a tag rather than a branch. It checks that the corpus is not a
submodule, and it warns about absolute home-directory paths. It exits nonzero on any failure, so
it can gate CI.</p>

<h2 id="adopting-it-without-breaking-anything">Adopting it without breaking anything</h2>

<p>An existing repository already has working code, frozen results and gates that pass, and adopting
the protocol must not break any of them. Adoption is additive first: add the manifest and point
its entries at wherever things already live, add the kind line and the research register, install
the kit, and run the repository’s own gate. It must pass exactly as it did before. Moving folders
into their default places is optional and comes later, one commit per move.</p>

<p>Analyses frozen under an earlier preregistration system stay exactly as they were frozen. They are
listed in the experiment register with a note saying which system froze them, and the kit is used
for new experiments only. Converting a frozen record would change the very thing the freeze exists
to protect.</p>

<h2 id="where-it-comes-from-and-what-it-is-not">Where it comes from, and what it is not</h2>

<p>The rules draw on published practice on organising computational projects, scientific computing,
reproducible research, preregistration, adaptive preregistration for model-based research, and
research software as a citable output. The protocol lists those sources in its
<a href="https://github.com/polarizetech/scientific-research-scaffold/blob/main/PROTOCOL.md#where-this-comes-from">closing section</a>.
No published protocol was found for laying out a whole research programme across repositories. The
split into studies, simulators and one shared corpus is an extrapolation from that practice, and it
should be read as one.</p>

<h2 id="using-it">Using it</h2>

<p>The protocol is licensed CC BY 4.0 and the code MIT. It needs Python 3.9 or later and git, and
nothing else. To use it for your own work, fork it and write a profile naming your own corpus,
preregistration kit, design system and workbench; any of them can be left empty. The first release,
v0.1.0, is on GitHub at
<a href="https://github.com/polarizetech/scientific-research-scaffold">polarizetech/scientific-research-scaffold</a>.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[Why the work here is split into studies, simulators and one shared research corpus, and scientific-research-scaffold, the small CLI that sets new repositories up in that shape and checks existing ones against it.]]></summary></entry><entry><title type="html">A spiking network built to lose: what it would and would not remember</title><link href="https://polarize.tech/blog/a-network-built-to-lose/" rel="alternate" type="text/html" title="A spiking network built to lose: what it would and would not remember" /><published>2026-09-25T07:00:00-06:00</published><updated>2026-09-25T07:00:00-06:00</updated><id>https://polarize.tech/blog/a-network-built-to-lose</id><content type="html" xml:base="https://polarize.tech/blog/a-network-built-to-lose/"><![CDATA[<p>Everything below is a result about a computer model with chosen parameters. None of it is a
measurement of a brain, an animal or a cell, and the tier says so. The code, every preregistered
plan and every raw output are in a public repository:
<a href="https://github.com/polarizetech/neural-memory">polarizetech/neural-memory</a>.</p>

<h2 id="the-question">The question</h2>

<p>Could a network of spiking neurons, with synapses that tag and consolidate the way published
models describe, store several sounds at once and play them back later from its own activity?</p>

<p>The project was set up to fail visibly. Every mechanism has an off switch, every result sits
beside the same run with that mechanism removed, and a plain reservoir network is always run
alongside as a baseline.</p>

<h2 id="the-tape-did-not-work">The tape did not work</h2>

<p>Sound went in readably: a linear decoder recovered the input envelopes from the network’s activity
while it listened. Nothing came back out. At every delay, and with every way of prompting recall
that was tried, the decoded output matched the stored sound no better than it matched sounds the
network had never heard. The plain reservoir encoded better.</p>

<p>An early result looked like a partial success: which stored sound was dominant at a given moment could
be read from the order in which cells fired, 77% of the time where shuffled labels reached 57%. A later
code review showed that ordering was measured while the sound was playing and was driven mostly by the
input itself. It says the cells followed the input, not that the network kept anything.</p>

<p>The weight changes explain the failure. What the network wrote into its synapses was set by which
cells happened to fire hardest, not by what they heard. A weight change predicted from any of
twenty sounds the network never heard matched the real one as well as the played sound’s did.</p>

<h2 id="habituation-as-memory">Habituation as memory</h2>

<p>The project then asked a smaller question. Repeated sounds evoke smaller responses. Is that
fading a memory of the particular sound, or just fatigue?</p>

<p>Four mechanisms were compared in a small auditory network, each with its own switch:</p>

<ul>
  <li>depletion of the input synapses;</li>
  <li>depression of a synapse only when the receiving cell also fires;</li>
  <li>inhibition that learns, using a rule of the form published in <sup class="ui-cite"><a href="#ref-vogels2011" id="cite-vogels2011-4" title="Inhibitory Plasticity Balances Excitation and Inhibition in Sensory Pathways and Memory Networks">4</a></sup>;</li>
  <li>receptor removal and replacement, as modelled for a single-celled organism <sup class="ui-cite"><a href="#ref-rajan2025" id="cite-rajan2025-1" title="A receptor-inactivation model for single-celled habituation in Stentor coeruleus">1</a></sup>.</li>
</ul>

<p>Two experiments were preregistered: predictions, pass criteria and code were fixed in git before
anything ran. Both closed as failures, because some predictions missed. What they showed:</p>

<p><strong>Depletion kept no sound-specific memory.</strong> At no delay, from 2 seconds to 90 minutes, did it
suppress the trained sound more than a different one. The main reason is in the ear model. At a
normal listening level, the least-similar of twenty random test sounds still overlapped the
trained one by 0.59 in the simulated auditory nerve, on a scale where 1 is identical. Depleting
shared input fibres cannot tell the two apart.</p>

<p><strong>Only plasticity gated by the receiving cell was specific.</strong> Depression that needed the
receiving cell to fire picked out the trained sound 30 minutes later. The learned inhibition
suppressed the trained sound too, and removing that inhibitory pathway undid all of it. Its
specificity was limited by the same 0.59 overlap.</p>

<h2 id="a-model-that-drains-where-the-cell-does-not">A model that drains where the cell does not</h2>

<p>The fourth mechanism reproduces a published model of habituation in <em>Stentor</em>, a single-celled
organism. In that model, stimulated receptors are pulled inside the cell and then recycled or
destroyed, and new receptors are made continuously <sup class="ui-cite"><a href="#ref-rajan2025" id="cite-rajan2025-1" title="A receptor-inactivation model for single-celled habituation in Stentor coeruleus">1</a></sup>. In
real cells, blocking protein synthesis made habituation faster and memory longer, while untrained
cells given the same drug kept responding normally <sup class="ui-cite"><a href="#ref-rajan2026" id="cite-rajan2026-2" title="Molecular pathways for learning in the single-cell Stentor coeruleus">2</a></sup>.</p>

<p>Run with the published model’s own rates, and the paper’s time step read as one minute (the paper
states no unit), the block did not do that here:</p>

<ul>
  <li>untrained responses fell by 32% after 20 minutes and 79% after 90 minutes;</li>
  <li>the extra memory the block produced was at most 1.4 points of suppression.</li>
</ul>

<p>The published model has basal loss of surface receptors, so a synthesis block drains untrained
cells in the model too. There the drain is hidden by a hard threshold: a cell far above its
contraction threshold keeps contracting while its receptors run down. A readout without that
threshold, like this network’s, exposes it. <strong>In this model, the cell’s normal untrained response
depends on the threshold, not on the receptor pool.</strong> Whether that holds in the organism is a
question for an experiment, not this simulation.</p>

<h2 id="spacing-did-not-help">Spacing did not help</h2>

<p>In roundworms trained at 60-second intervals, long-term habituation followed training split into
blocks with hour-long rests.
Training all at once lowered next-day responses too, but only the spaced group responded
significantly less on the second day than on the first <sup class="ui-cite"><a href="#ref-beck1997" id="cite-beck1997-3" title="Long-term habituation is produced by distributed training at long ISIs and not by massed training or short ISIs inCaenorhabditis elegans">3</a></sup>.</p>

<p>None of the mechanisms reproduced a spacing benefit. With the same number of presentations, spaced
training left less suppression than massed training in the receptor and learned-inhibition models,
and no difference for depletion. (The excitatory-depression model also favoured massed training, but
a later review found its untrained comparison network drifts during a long schedule, so that
comparison is confounded.) Each mechanism has a single decay rate, so earlier blocks simply fade. A spacing effect seems to need a
second, slower consolidation stage that none of these models has.</p>

<h2 id="what-would-change-these-conclusions">What would change these conclusions</h2>

<ul>
  <li>A test pair with genuinely low overlap in the auditory nerve (below about 0.2), at which
depletion does keep a specific trace. The overlap limit is a property of this ear model at this
level, not a general law.</li>
  <li>Adding a hard response threshold to the receptor model’s readout and finding the untrained
response still drains.</li>
  <li>A single-timescale mechanism that nonetheless favours spaced training.</li>
</ul>

<p>The project is paused here. Its findings, defects and the next experiments each would need are
listed in the repository.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[A small, biologically grounded network was asked to store sounds and play them back. It could not. Along the way it showed which habituation mechanisms keep a stimulus-specific memory, and where a published single-cell model parts ways with the cell it describes.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/golgi-pyramidal-neuron.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/golgi-pyramidal-neuron.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">Adaptive preregistration: predict first, then run the code</title><link href="https://polarize.tech/blog/adaptive-preregistration-predict-first-then-run-the-code/" rel="alternate" type="text/html" title="Adaptive preregistration: predict first, then run the code" /><published>2026-09-24T12:00:00-06:00</published><updated>2026-09-24T12:00:00-06:00</updated><id>https://polarize.tech/blog/adaptive-preregistration-predict-first-then-run-the-code</id><content type="html" xml:base="https://polarize.tech/blog/adaptive-preregistration-predict-first-then-run-the-code/"><![CDATA[<p>A simulation can be tuned until it agrees with you. Each choice is small: a seed, a threshold,
an analysis window, a parameter nobody measured. None of them looks like cheating, and
together they can manufacture any result.</p>

<p>Software makes this cheap. A new variant costs seconds, and the run that finally agrees looks
exactly like one that was planned. The fix is the same one experimental science uses: write
down what would count as success before looking, and keep a record that shows the order things
happened in.</p>

<p>This is the protocol used for model experiments here. It adapts published work on adaptive
preregistration for model-based research and on reporting deviations from a preregistered
plan. It is written for simulations, analysis pipelines and research software, whoever or
whatever is doing the running. The full protocol, with its sources and how deeply each was read,
is in the <a href="https://github.com/polarizetech/adaptive-preregistration/blob/main/modules/prereg/protocols/PREREG_PROTOCOL.md">protocol document</a>.</p>

<h2 id="the-rules">The rules</h2>

<ul>
  <li><strong>A claim, or an exploratory label.</strong> Every piece of work, whether an app, a simulation, a tool
or a calculator, starts with a falsifiable claim, settled in the author’s own words together
with what would count against it. Work the author marks as exploratory may be built without
one: it is recorded and labelled as exploratory, nothing it shows counts as a finding, and it
gets its claim before its first experiment is preregistered.</li>
  <li><strong>No run before the preregistration.</strong> A run whose result a report will cite may not
execute until <code class="language-plaintext highlighter-rouge">PREREG.md</code> is complete and tagged.</li>
  <li><strong>The environment is part of the plan.</strong> The preregistration names the model version it runs
against, and a lockfile pins every dependency. Adding a dependency afterwards is a deviation.</li>
  <li><strong>Failure closes the version; it does not edit it.</strong> A failed experiment is closed with its
failure written up, and the next attempt gets a new experiment ID. Every ID stays in a
registry, so a pass after earlier failures is reported as one attempt among several.</li>
  <li><strong>Every departure from the plan is logged,</strong> dated, with whether the outcome was known at
the time.</li>
  <li><strong>Exploratory work is quarantined.</strong> Anything not in the plan lives in <code class="language-plaintext highlighter-rouge">exploratory/</code> and is
labelled exploratory everywhere it is mentioned.</li>
</ul>

<h2 id="what-makes-it-adaptive">What makes it adaptive</h2>

<p>Modelling is iterative, and a protocol that forbids iteration gets ignored. The rule is about
order, not rigidity.</p>

<ul>
  <li>A plan may change between stages. Each stage says in advance which result leads to which
change. The change is committed and tagged <em>before</em> the run it governs, and logged with the
outcome marked as not yet known.</li>
  <li>A plan may also change after a result is seen. It is still logged, with the outcome marked as
known, and it can never be used to convert a fail into a pass.</li>
  <li>An experiment that fails stays in the record. Nothing is deleted or cleaned up.</li>
</ul>

<h2 id="what-the-preregistration-contains">What the preregistration contains</h2>

<p>Eleven sections, all written before any scoring run:</p>

<ul>
  <li>the question, as one mechanistic sentence;</li>
  <li>risky, numeric, directional predictions, each with the result that would count against it;</li>
  <li>pass and fail thresholds for each estimated quantity, with its uncertainty: a pass means the
interval clears the threshold, not just the point estimate;</li>
  <li>the outcomes that would close the line of work;</li>
  <li>the model specification, with every parameter tagged as taken from literature, derived, or
arbitrary;</li>
  <li>the design: conditions, a fixed list of seeds, controls, exclusion rules, a justified number of
runs with a stopping rule, and a sensitivity analysis for every arbitrary parameter. A pass that
flips to a fail anywhere in a preregistered range is reported as not robust;</li>
  <li>the environment, down to the execution backend and thread count, because the same seed does
not give the same result everywhere;</li>
  <li>what the authors already knew: which target data they had seen, and which targets the model
was calibrated to rather than tested against;</li>
  <li>any adaptive stages, every decision the specification left open, and how the plan was
timestamped.</li>
</ul>

<p>The results file answers the plan line by line. It also has to list the patterns the model
failed to reproduce, what only worked because it was tuned, and the result of every control.</p>

<h2 id="the-record">The record</h2>

<p>Git holds the ordering. Each milestone is an annotated tag:</p>

<table>
  <thead>
    <tr>
      <th>Tag</th>
      <th>Marks</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td><code class="language-plaintext highlighter-rouge">model-vX.Y.Z</code></td>
      <td>a change to the model that alters its output</td>
    </tr>
    <tr>
      <td><code class="language-plaintext highlighter-rouge">&lt;EID&gt;-prereg</code></td>
      <td>the complete plan, lockfile and configuration</td>
    </tr>
    <tr>
      <td><code class="language-plaintext highlighter-rouge">&lt;EID&gt;-interim-N</code></td>
      <td>a plan revision, before the run it governs</td>
    </tr>
    <tr>
      <td><code class="language-plaintext highlighter-rouge">&lt;EID&gt;-run</code></td>
      <td>the outputs and the results file</td>
    </tr>
    <tr>
      <td><code class="language-plaintext highlighter-rouge">&lt;EID&gt;-closed</code></td>
      <td>the end of the experiment, pass or fail</td>
    </tr>
  </tbody>
</table>

<p>Each experiment gets its own branch and draft pull request. Tagging a milestone posts a receipt
to the pull request with the commit and a checksum of the plan and the lockfile. The comment’s
timestamp comes from the hosting service, not from the machine that made the commit, so it shows
the plan existed by then.</p>

<h2 id="rules-for-whoever-runs-it">Rules for whoever runs it</h2>

<p>The same rules apply to a person at the keyboard, a script, or a coding assistant.</p>

<ul>
  <li>Before running anything citable, confirm the plan is complete and tagged. If it is not,
write it and stop for someone else to review.</li>
  <li>Never edit the plan after it is tagged. Changes go in the deviations table.</li>
  <li>Asked to “make it pass” or “try a few values and keep the best”, do the runs under
<code class="language-plaintext highlighter-rouge">exploratory/</code> and say plainly that they are not preregistered evidence.</li>
  <li>State every open decision before the run that depends on it.</li>
  <li>In every report, state how deeply each source was read: full text, abstract, background
knowledge, or supplied by the user.</li>
  <li>If anyone asks to skip a step, write the skip into the deviations table first, with the
outcome-known field filled in honestly.</li>
</ul>

<h2 id="how-it-reaches-every-project">How it reaches every project</h2>

<p>The protocol is maintained in one public repository,
<a href="https://github.com/polarizetech/adaptive-preregistration">KIT Adaptive Preregistration</a>, and
installed into each project with a small command-line tool, <code class="language-plaintext highlighter-rouge">kit_ap</code>. It copies the protocol documents and tools into the project’s
<code class="language-plaintext highlighter-rouge">.agents/</code> folder and records the exact version in a lockfile. It also writes the rules into
<code class="language-plaintext highlighter-rouge">AGENTS.md</code>, so coding assistants working in the repository read the same rules a person
would.</p>

<p>Some of the rules are backed by code rather than left to good intentions:</p>

<ul>
  <li>an optional commit guard refuses outputs for an experiment that has no preregistration tag,
and refuses any change to a plan after it is tagged (like any git hook, it can be bypassed);</li>
  <li>where the tools support hooks, the current experiment’s plan status is surfaced on every
session;</li>
  <li>at the start of a session, the project checks whether the protocol has changed upstream, and
reports it without updating on its own.</li>
</ul>

<h2 id="limits">Limits</h2>

<p>This protects the record, not the idea. A well-preregistered experiment on a wrong model is
still wrong.</p>

<p>A local git history is not tamper-evident: tags can be moved unless they are signed and
protected on the host. The pull-request receipt is a third-party clock but not an archive, since
comments can be edited, and it can’t show that nothing ran before the plan. For outside
credibility, the preregistration tag should also be deposited with an archive, and the plan should
say which.</p>

<p>Nothing stops a new attempt after a failure. The registry only makes the attempts visible, so a
reader can weigh a pass against them.</p>

<p>Most of the protocol is rules that people and tools are asked to follow. Only the commit guard
and the hooks enforce anything, and the hooks only in tools that run them. The rest relies on the
record making a violation visible afterwards.</p>

<h2 id="update--2026-09-24">Update — 2026-09-24</h2>

<p>The kit’s repository is now public and linked from the section on how the protocol reaches
each project.</p>

<p>After a methods review, the protocol was tightened, and this post was revised to match. It now
describes: the registry of attempts, uncertainty in the pass criteria, a justified run count, a
sensitivity rule fixed in advance, a section on prior knowledge and calibration (eleven sections,
previously ten), and decision rules for adaptive stages. The limits section now says more about
what the record can and can’t prove. Previously the post said a pass that depends on an arbitrary
parameter does not count; the rule is now that a pass which flips within a preregistered range is
reported as not robust.</p>

<h2 id="update--2026-09-25">Update — 2026-09-25</h2>

<p>Recording coding-assistant conversations is no longer part of the protocol, and the kit no longer
installs it. The post previously said each prompt and reply was posted to the experiment’s pull
request and committed beside it; that paragraph and the matching line under “How it reaches every
project” were removed. The kit’s repository was also renamed, and its links here point to the new
address.</p>

<h2 id="update--2026-09-30">Update — 2026-09-30</h2>

<p>The protocol gained a rule that comes before the others: every piece of work starts with a
falsifiable claim, stated with what would count against it, before anything is built. Settling it
means saying what the claim’s terms mean, how it will be measured, the smallest effect that would
matter, and what a test of it assumes. The section above was previously titled “The five rules”.
Preregistration now also works per piece of work: a project holding several apps, simulations,
tools or calculators gives each its own claim, experiments and versions.</p>

<h2 id="update--2026-10-07">Update — 2026-10-07</h2>

<p>The first rule changed. It previously said every piece of work starts with a falsifiable claim
before anything is built. Work can now be marked exploratory instead: it is built from a short
note of what is being built and what is already known, it is labelled exploratory, and nothing it
shows counts as a finding. Its claim is settled before its first experiment is preregistered.
Settling a claim before building now means stating the claim and what would count against it.
What its terms mean, how it will be measured, the smallest effect that would matter and what a
test of it assumes are stated in the first preregistration, not before building.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[A protocol for simulations and research software in which the predictions, the pass criteria and the environment are fixed in git before anything a report will cite is allowed to run.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/darwin-notebook-b-tree.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/darwin-notebook-b-tree.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">A RAG tool that keeps the model in check</title><link href="https://polarize.tech/blog/a-rag-tool-that-keeps-the-model-in-check/" rel="alternate" type="text/html" title="A RAG tool that keeps the model in check" /><published>2026-09-24T07:00:00-06:00</published><updated>2026-09-24T07:00:00-06:00</updated><id>https://polarize.tech/blog/a-rag-tool-that-keeps-the-model-in-check</id><content type="html" xml:base="https://polarize.tech/blog/a-rag-tool-that-keeps-the-model-in-check/"><![CDATA[<p>Retrieval-augmented generation is not a citation system by itself. It gives a model more text;
the protocol has to make that text accountable.</p>

<p>This is the method used in
<a href="https://github.com/polarizetech/retrieval-augmented-generation">KIT Retrieval-Augmented Generation</a>:</p>

<h2 id="pipeline">Pipeline</h2>

<ul>
  <li><strong>Plan:</strong> turn the question into sub-questions, search terms and falsification queries.</li>
  <li><strong>Discover:</strong> search the available literature providers and record providers that did not answer.</li>
  <li><strong>Acquire:</strong> fetch accessible full text through the paper library.</li>
  <li><strong>Index:</strong> split the text into passages with stable evidence IDs.</li>
  <li><strong>Retrieve and rerank:</strong> combine lexical and semantic search, then select the passages to inspect.</li>
  <li><strong>Extract:</strong> record the passage, source, direction, population, study role and a verbatim quote.</li>
  <li><strong>Synthesise:</strong> let the model draft only from evidence IDs that were actually retrieved.</li>
  <li><strong>Critique:</strong> search again for null results, opposing results and failed replications; do not merely
ask the model to reconsider its own draft.</li>
  <li><strong>Verify:</strong> check quotes and numbers in code, then judge each claim against its cited passage.</li>
  <li><strong>Render and log:</strong> print bibliographic metadata from stored records and save the searches,
passages, model versions, verdicts and limits.</li>
</ul>

<h2 id="rules">Rules</h2>

<ul>
  <li>The model fills bounded, schema-constrained forms. Code controls the sequence.</li>
  <li>A paper’s existence and a passage’s support for a claim are separate checks.</li>
  <li>A quote must occur in the stored passage.</li>
  <li>A number in a claim must occur in its cited evidence, with a matching unit where the field
declares units.</li>
  <li>A citation must be an evidence ID from the run; the model does not type the bibliography.</li>
  <li>A passage describing another paper is a pointer, not independent first-hand evidence.</li>
  <li>Verifier disagreement is reported as disputed, not averaged away.</li>
  <li>Failed claims are removed and counted in the limits.</li>
  <li>“No opposing result was retrieved” is a statement about the search, not about the literature.</li>
  <li>Retrieved papers are data, not instructions. Text addressed to an AI reader is excluded when
detected.</li>
  <li>A run’s own output is never indexed as a source for a later run.</li>
</ul>

<h2 id="extending-it">Extending it</h2>

<p>The engine is domain-neutral. A domain package supplies the rules that the engine cannot know:</p>

<ul>
  <li>which study designs count as evidence;</li>
  <li>which sources are authoritative;</li>
  <li>which units are equivalent;</li>
  <li>which species, preparation or outcome gaps limit generalisation.</li>
</ul>

<p>The domain is recorded in the run log. Adding a neuroscience, cardiovascular or vestibular
extension changes the field rules without forking retrieval, verification or logging.</p>

<h2 id="limits">Limits</h2>

<p>This does not make a language model truthful. It reduces the paths by which unsupported claims
enter an answer and makes the remaining uncertainty visible.</p>

<p>It does not recover missing figures or supplements, make closed papers available, or guarantee
that a verifier is right. When another model writes the answer through the repository’s MCP
evidence tools, only the deterministic checks apply (evidence ids, quotes and numbers); whether a
passage supports a claim is judged only inside the pipeline. A useful result can still be
<strong>insufficient evidence</strong>.</p>

<h2 id="update--2026-09-24">Update — 2026-09-24</h2>

<p>The repository is now public and linked above. Before publishing, the code was brought into line
with this description: a claim whose number does not occur in its source is now removed rather
than marked disputed, and the MCP evidence tools now apply the quote and number checks too.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[A short, evidence-first protocol for using retrieval-augmented generation without letting a language model turn an unsupported answer into a finding.]]></summary></entry><entry><title type="html">Twelve ways to catch a green crab</title><link href="https://polarize.tech/blog/twelve-ways-to-catch-a-green-crab/" rel="alternate" type="text/html" title="Twelve ways to catch a green crab" /><published>2026-09-16T09:00:00-06:00</published><updated>2026-09-16T09:00:00-06:00</updated><id>https://polarize.tech/blog/twelve-ways-to-catch-a-green-crab</id><content type="html" xml:base="https://polarize.tech/blog/twelve-ways-to-catch-a-green-crab/"><![CDATA[<p>This is a case study of a search that mostly returned no.</p>

<p>The subject is the European green crab (<em>Carcinus maenas</em>), an invasive
portunid established on the coast of British Columbia. The question I set out
with was narrow and, I thought, tractable: <strong>is there any signal a green crab
can detect that a native crab cannot</strong> — because if there is, you can build it
into a trap and catch one species without catching the other.</p>

<p>Twelve routes were screened. <strong>Ten are closed. One is real but unreachable with
equipment I can obtain. Two survive, and neither of them is a device.</strong></p>

<p>None of this is novel. Every closure came from applying published work or
undergraduate physics to a specific question, and in one case the thing I
declared missing from the literature turned out to have been published, with
public code, four months earlier. <strong>The value here, if there is any, is the
shape of the negative results and the order they arrived in</strong> — so I am writing
it down in public rather than leaving it in a private repository. If any of it
saves somebody a month, take it.</p>

<h2 id="the-constraint-that-governs-everything">The constraint that governs everything</h2>

<p><strong>A green crab trap that also catches Dungeness crab is worse than no trap.</strong>
Dungeness supports British Columbia’s most valuable crab fishery, and juvenile
Dungeness share estuarine nursery habitat with juvenile green crab. So
“attracts green crab” was never sufficient. The requirement was always
<strong>differential</strong> — something the target detects and the bycatch does not.</p>

<p>That single constraint is what killed most of the twelve.</p>

<h2 id="the-ledger">The ledger</h2>

<table>
  <thead>
    <tr>
      <th>#</th>
      <th>Route</th>
      <th>Verdict</th>
      <th>What closed it</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td>1</td>
      <td><strong>Electric prey mimicry</strong> — a lure imitating prey bioelectric fields</td>
      <td><strong>CLOSED</strong></td>
      <td>Prey fields are a contact cue even for a shark; no crustacean electroreceptor has been identified</td>
    </tr>
    <tr>
      <td>2</td>
      <td><strong>Magnetic</strong> — exploit a reported sex-specific field response</td>
      <td><strong>OPEN, unreachable</strong></td>
      <td>Real result, unreplicated, no located transducer, and an unresolved thermal confound</td>
    </tr>
    <tr>
      <td>3</td>
      <td><strong>Substrate vibration</strong> from buried prey</td>
      <td><strong>CLOSED</strong></td>
      <td>Every catalogued prey sound sits outside the crab’s measured mechanoreceptor band</td>
    </tr>
    <tr>
      <td>4</td>
      <td><strong>Water-borne prey sound</strong></td>
      <td><strong>CLOSED</strong></td>
      <td>Near-field falloff and displacement arithmetic put it at centimetres</td>
    </tr>
    <tr>
      <td>5</td>
      <td><strong>Acoustic reproductive interference</strong> — mask mating signals</td>
      <td><strong>CLOSED</strong></td>
      <td>The water is too shallow to propagate the relevant frequencies at all</td>
    </tr>
    <tr>
      <td>6</td>
      <td><strong>Chemical prey odour</strong></td>
      <td><strong>WORKS, NOT SELECTIVE</strong></td>
      <td>Out-ranges every mechanical cue by orders of magnitude, and every crab there smells it</td>
    </tr>
    <tr>
      <td>7</td>
      <td><strong>Sex pheromone lure</strong></td>
      <td><strong>WORKS, NOT SELECTIVE ENOUGH</strong></td>
      <td>Attracts males of the target — and the bycatch problem is unaddressed</td>
    </tr>
    <tr>
      <td>8</td>
      <td><strong>Predator cue</strong> — flush crabs out of refuge into gear</td>
      <td><strong>CLOSED</strong></td>
      <td>Requires a cue that moves the target and not the natives; same failure as 6</td>
    </tr>
    <tr>
      <td>9</td>
      <td><strong>Parasite biocontrol</strong></td>
      <td><strong>CLOSED, decisively</strong></td>
      <td>Host-specificity testing against native Pacific crabs is the standing answer</td>
    </tr>
    <tr>
      <td>10</td>
      <td><strong>Native predator recovery</strong></td>
      <td><strong>OPEN, not a lever</strong></td>
      <td>One landscape-scale success exists; its agent is absent from the relevant water</td>
    </tr>
    <tr>
      <td>11</td>
      <td><strong>Gear</strong> — trap type and entrance geometry</td>
      <td><strong>SURVIVES</strong></td>
      <td>Largest demonstrated effect anywhere in this exercise</td>
    </tr>
    <tr>
      <td>12</td>
      <td><strong>Place and schedule</strong> — where and when the gear is set</td>
      <td><strong>SURVIVES</strong></td>
      <td>Two independent axes with real supporting evidence</td>
    </tr>
  </tbody>
</table>

<p><strong>Five independent lines of work converged on the bottom two rows.</strong> That
convergence is the single most useful thing the exercise produced, and it took
about eight closures to get there.</p>

<hr />

<h2 id="where-it-started-the-electromagnetic-branch">Where it started: the electromagnetic branch</h2>

<p>The project began with a specific published result: juvenile green crabs
exposed to static magnetic fields at strengths relevant to submarine power
cables showed a <strong>sex-specific</strong> response, with females spending more time in
exposed zones and males showing no consistent
preference.</p>

<aside class="ui-source" id="ref-james2025">
  <a class="ui-source__link" href="https://doi.org/10.1021/acs.estlett.5c00862" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Female Crabs Are More Sensitive to Environmentally Relevant Electromagnetic Fields from Submarine Power Cables</span>
      <span class="ui-source__meta">
        James et al.
        · 2025 · Environmental Science &amp; Technology Letters
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>That is exactly the shape of thing the constraint above demands — a
differential response, in the target species, in a channel you can generate
with a coil. It is why this project exists at all.</p>

<p><strong>Three things had to be true for it to become a trap, and I could establish
none of them.</strong></p>

<p><strong>First, a mechanism.</strong> No transducer has been located. The obvious comparison
is the spiny lobster, the standard invertebrate magnetoreception
system
— but the receptor cells have not been located and characterised in that animal
either. Mapping a mechanism from one order of crustaceans onto another, across
more than two hundred million years of divergence, when the source species’
anatomy is itself unresolved, produces a hypothesis wearing borrowed
credibility.</p>

<aside class="ui-source" id="ref-lohmann1984">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.113.1.29" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Magnetic Remanence in the Western Atlantic Spiny Lobster, Panulirus Argus</span>
      <span class="ui-source__meta">
        Lohmann
        · 1984 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-boles2003">
  <a class="ui-source__link" href="https://doi.org/10.1038/nature01226" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">True navigation and magnetic maps in spiny lobsters</span>
      <span class="ui-source__meta">
        Boles et al.
        · 2003 · Nature
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-ernst2016">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.136036" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Effect of magnetic pulses on Caribbean spiny lobsters: implications for magnetoreception</span>
      <span class="ui-source__meta">
        Ernst et al.
        · 2016 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Second, the field map has to reproduce.</strong> It does not. No coil geometry I
could construct, at any separation or tank bearing, reproduces the published
zone table — best fit was 61% RMS error. That is a correspondence-with-the-authors
problem, not a finding, and it is recorded as one.</p>

<p><strong>Third, the confound.</strong> Helmholtz coils dissipate heat and crabs are
thermotactic. Working the published geometry through a thermal model gives,
at the strongest field, roughly <strong>20 W dissipated, a 0.58 K gradient across the
tank and a 0.30 K bulk rise</strong> — small, but not obviously below what an animal
can detect, and I could not find a behavioural thermal-discrimination threshold
for this species to compare it against.</p>

<p><strong>One thing argues against the thermal explanation, and it is worth stating
because it cuts my way and I nearly missed it.</strong> Ohmic heating scales with the
square of the current, so the confound is about ten times larger at the
strongest field than at the intermediate one — while the reported attraction
was <em>strongest at the intermediate field</em>. <strong>The confound and the effect run in
opposite directions.</strong> A thermocouple in the tank would settle it, and it is the
cheapest experiment anywhere in this review.</p>

<p><strong>Verdict: open, and unreachable here.</strong> The claim is untouched. What closes it
is a replication with a sham coil and a temperature log, which needs a facility
and animals I do not have.</p>

<h3 id="and-the-electric-branch-is-closed-which-is-a-different-answer">And the electric branch is closed, which is a different answer</h3>

<p>The original premise was electric, not magnetic — a lure imitating the
bioelectric field of buried prey. It is closed on two independent grounds.</p>

<p><strong>The physics.</strong> Prey bioelectric fields were measured at <strong>microvolt scale
with the electrode less than a millimetre from the tissue</strong>, and the authors
state plainly that the voltage from invertebrates <strong>was too weak to record away
from the source</strong>. Run through a
shark’s own measured sensitivity, a natural prey field is readable at a few
centimetres. A crab is not a shark.</p>

<aside class="ui-source" id="ref-bedore2013">
  <a class="ui-source__link" href="https://doi.org/10.1086/669973" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Bioelectric Fields of Marine Organisms: Voltage and Frequency Contributions to Detectability by Electroreceptive Predators</span>
      <span class="ui-source__meta">
        Bedore et al.
        · 2013 · Physiological and Biochemical Zoology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p><strong>The biology.</strong> No electroreceptor has been identified in any crustacean, and
none has been sought in green crab. A behavioural sensitivity figure exists for
a freshwater crayfish — a surrogate,
from a different order, in fresh water.</p>

<aside class="ui-source" id="ref-patullo2010">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.039073" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Making sense of electrical sense in crayfish</span>
      <span class="ui-source__meta">
        Patullo et al.
        · 2010 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>That is not a modelling gap. It is the state of the field</strong>, and the honest
output was to say so rather than to model around it.</p>

<p><strong>And the welfare evidence points the same way.</strong> Green crabs have nociceptors in
every soft tissue tested, and they
<strong>learn to avoid a place where they receive electric shock</strong> — some dropping a
wired leg even though the voltage was set below the single-shock level that
causes it. That was contact current, not a
field in water, so it sets no threshold. But it means an electric lure for this
animal should be expected to repel as well as attract.</p>

<aside class="ui-source" id="ref-kasiouras2024">
  <a class="ui-source__link" href="https://doi.org/10.3390/biology13110851" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Putative Nociceptive Responses in a Decapod Crustacean: The Shore Crab (Carcinus maenas)</span>
      <span class="ui-source__meta">
        Kasiouras et al.
        · 2024 · Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-magee2013">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.072041" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Shock avoidance by discrimination learning in the shore crab (Carcinus maenas) is consistent with a key criterion for pain</span>
      <span class="ui-source__meta">
        Magee et al.
        · 2013 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<hr />

<h2 id="prey-signalling-vibration-and-sound">Prey signalling: vibration and sound</h2>

<p>If the crab cannot be lured electrically, the next question is what its prey
actually broadcasts, and whether a trap can imitate it.</p>

<p><strong>The receiver side is better documented than I expected.</strong> There is a real
transfer function for the mouthpart setae — displacement thresholds, and the
coding: spike count scales with displacement amplitude, interspike interval
with velocity. <strong>That paper is also
where I made my first substantive error</strong> (below): those setae are <em>tactile</em>
receptors for handling prey, not distance detectors, and I spent a while
scoring far-field stimuli against them.</p>

<aside class="ui-source" id="ref-garm2005">
  <a class="ui-source__link" href="https://doi.org/10.1007/s00227-005-0020-7" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Mechanosensory properties of the mouthpart setae of the European shore crab Carcinus maenas</span>
      <span class="ui-source__meta">
        Garm
        · 2005 · Marine Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>The organ that matters for substrate vibration is a joint organ in the walking
leg, described in green crab itself,
with a measured band. Water motion is a different receptor
again; the behavioural response of
intact animals to substrate vibration has been tested
directly; decapod acoustic detection has
been reviewed as a field; an
evoked-potential study in the American lobster asks which organ is
responsible; and a consolidated review
of green crab sensory biology exists.</p>

<aside class="ui-source" id="ref-burke1954">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.31.1.127" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">An Organ for Proprioception and Vibration Sense in Carcinus Maenas</span>
      <span class="ui-source__meta">
        Burke
        · 1954 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-tautz1980">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.88.1.351" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">The Detection of Waterborne Vibration by Sensory Hairs on the Chelae of the Crayfish</span>
      <span class="ui-source__meta">
        Tautz et al.
        · 1980 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-aimon2021">
  <a class="ui-source__link" href="https://doi.org/10.1016/j.envpol.2021.117148" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Anthropogenic underwater vibrations are sensed and stressful for the shore crab Carcinus maenas</span>
      <span class="ui-source__meta">
        Aimon et al.
        · 2021 · Environmental Pollution
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-popper2001">
  <a class="ui-source__link" href="https://doi.org/10.1007/s003590100184" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Acoustic detection and communication by decapod crustaceans</span>
      <span class="ui-source__meta">
        Popper et al.
        · 2001 · Journal of Comparative Physiology A: Sensory, Neural, and Behavioral Physiology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-jzquel2021">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.240747" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Sound detection by the American lobster (Homarus americanus)</span>
      <span class="ui-source__meta">
        Jézéquel et al.
        · 2021 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-jury2024">
  <a class="ui-source__link" href="https://doi.org/10.1016/B978-0-323-99694-5.00004-0" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Sensory biology and behaviour</span>
      <span class="ui-source__meta">
        Jury et al.
        · 2024 · Ecophysiology of the European Green Crab (Carcinus Maenas) and Related Species
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>The transmitter side is where it died.</strong> The reference dataset for benthic
invertebrate sound gives calibrated source levels for scallops, limpets,
urchins and crustaceans. Converting
each to particle displacement and solving for the crab’s threshold, <strong>not one
of the nine sources reaches a crab at more than millimetres</strong> — and every sound
in that dataset peaks between 5 and 49 kHz, while the analysis band was
filtered from 2 kHz upward.</p>

<aside class="ui-source" id="ref-coquereau2016">
  <a class="ui-source__link" href="https://doi.org/10.1007/s00227-016-2902-2" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Sound production and associated behaviours of benthic invertebrates from a coastal habitat in the north-east Atlantic</span>
      <span class="ui-source__meta">
        Coquereau et al.
        · 2016 · Marine Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p><strong>The corpus was built for hydrophone monitoring, not for prey detection, and
the crab’s band was removed before analysis.</strong> A null there is <em>unavailable</em>,
not absent, and the distinction is the whole point of recording it.</p>

<p>Two pieces of arithmetic govern all of this and are worth stating plainly,
because they close route 4 without any biology at all:</p>

<ul>
  <li><strong>Near-field falloff.</strong> A small oscillating body in water produces a field
falling off as 1/r³ if it oscillates back and forth. The cube law is brutal:
a thousand times more source amplitude buys ten times the range.</li>
  <li><strong>Displacement is not pressure.</strong> Particle displacement equals velocity
divided by 2πf, so for a given sound pressure a kilohertz signal carries far
less displacement than a hundred-hertz one. <strong>High-frequency sound is
displacement-poor, and crabs detect displacement.</strong></li>
</ul>

<p><strong>The one prey cue that survives is not a sound at all.</strong> Porewater pressure
signals generated by infaunal activity have been recorded directly in
sediment, and the irrigation timing of
three tellinid bivalves — including a Pacific Northwest clam that is real green
crab prey — has been measured in detail.
That is a slow hydraulic signal, and it is the only prey cue in this review with
a field detection range measured on relevant species.</p>

<aside class="ui-source" id="ref-wethey2005">
  <a class="ui-source__link" href="https://doi.org/10.2307/3593131" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Infaunal Hydraulics Generate Porewater Pressure Signals</span>
      <span class="ui-source__meta">
        Wethey et al.
        · 2005 · The Biological Bulletin
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-volkenborn2012">
  <a class="ui-source__link" href="https://doi.org/10.1357/002224012806770955" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Intermittent bioirrigation and oxygen dynamics in permeable sediments: An experimental and modeling study of three tellinid bivalves</span>
      <span class="ui-source__meta">
        Volkenborn et al.
        · 2012 · Journal of Marine Research
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<hr />

<h2 id="mating-pheromone-and-interference">Mating: pheromone, and interference</h2>

<p><strong>Chemistry out-ranges every mechanical cue by two to three orders of
magnitude.</strong> Modelled as a plume, prey odour reaches hundreds of metres where
the best mechanical cue reaches a couple. The receptor side has two
anatomically separate systems doing different jobs — olfaction on the
antennules, and contact chemoreception on the dactyls, where the gustatory
organs of this species have been characterised
electrophysiologically.</p>

<aside class="ui-source" id="ref-schmidt1989">
  <a class="ui-source__link" href="https://doi.org/10.1007/BF00193467" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Specificity and response characteristics of gustatory sensilla (funnel-canal organs) on the dactyls of the shore crab, Carcinus maenas (Crustacea, Decapoda)</span>
      <span class="ui-source__meta">
        Schmidt et al.
        · 1989 · Journal of Comparative Physiology A
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>The female sex pheromone has been the subject of an identification
study, and later work using it
produced the single most interesting behavioural result in this review: males
presented with a pheromone-treated dummy female showed a mating response 87% of
the time under ambient conditions and 40% under ship-noise playback, a
significant drop — <strong>while the time taken to respond to the pheromone did not
change significantly</strong>. Noise
interfered with completing the behaviour, not with detecting the signal. That
dissociation is worth more than either number alone.</p>

<aside class="ui-source" id="ref-hardege2011">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps09226" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Identification of a female sex pheromone in Carcinus maenas</span>
      <span class="ui-source__meta">
        Hardege et al.
        · 2011 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-rising2022">
  <a class="ui-source__link" href="https://doi.org/10.1371/journal.pone.0276889" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Anthropogenic noise may impair the mating behaviour of the Shore Crab Carcinus Maenas</span>
      <span class="ui-source__meta">
        Rising et al.
        · 2022 · PLOS ONE
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p><strong>So chemistry works, and that is the problem.</strong> It is the best-performing
channel in the whole review and it is the <em>least</em> selective one: a bait plume
is smelled by every crab in the basin. A pheromone lure is better — it targets
males of one species — but males are demographically close to irrelevant, and it
does nothing about Dungeness bycatch.</p>

<p><strong>Route 5, acoustic reproductive interference, closes on physics rather than on
biology, and cleanly.</strong> Shallow water is a waveguide with a cutoff frequency
below which no mode propagates at all. At the 0.5–5 m depths where these
animals actually mate, the cutoff is <strong>159–1594 Hz</strong> — above the signal band
you would need to mask. <strong>You cannot interfere with a signal in water that will
not carry your interference.</strong></p>

<hr />

<h2 id="the-selectivity-problem-stated-properly">The selectivity problem, stated properly</h2>

<p>By this point the pattern was clear enough to test directly, so I built a
screening tool: for a given stimulus, how much arrives at a receptor, in what
format, at what range — and a refusal when the number underneath does not
exist. <a href="/blog/green-crab-sensory-screening-tool/">That has its own write-up</a>.</p>

<p><strong>Its most useful output was a comparison that cannot be run.</strong></p>

<p>Across eight receptor channels and five species, green crab has measured values
in five channels and a described-but-unmeasured organ in two. For Dungeness
crab, red rock crab, graceful rock crab and yellow shore crab, I found <strong>two</strong>
measured thresholds, both in Dungeness and both behavioural — a detection
threshold for a prey extract and
salinity detection measured by antennular
flicking. Both are held at abstract
only, so those are descriptions of what was measured, not of what was found.</p>

<aside class="ui-source" id="ref-pearson1979">
  <a class="ui-source__link" href="https://doi.org/10.1016/0022-0981(79)90005-4" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Thresholds for detection and feeding behavior in the dungeness crab, Cancer magister (Dana)</span>
      <span class="ui-source__meta">
        Pearson et al.
        · 1979 · Journal of Experimental Marine Biology and Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-sugarman1983">
  <a class="ui-source__link" href="https://doi.org/10.2307/1351397" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Salinity Detection and Associated Behavior in the Dungeness Crab, Cancer magister</span>
      <span class="ui-source__meta">
        Sugarman et al.
        · 1983 · Estuaries
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Two filled cells out of thirty-two.</strong> And they do not make the comparison
runnable, because they are behavioural thresholds in grams per litre while
every green crab value is single-unit electrophysiology in micrometres. Putting
them in one row would be a category error, not a comparison.</p>

<p><strong>That is the state of the literature, not a gap in the modelling.</strong> Green crab
is a classic laboratory animal; the natives are commercially and ecologically
important animals whose sensory physiology has largely not been measured.</p>

<p><strong>And where the bands <em>are</em> known, they overlap.</strong> Every crab whose
mechanoreception has been measured peaks around 100 Hz. There is no frequency
at which you can shout at a green crab and not be heard by a Dungeness.</p>

<p>What <em>can</em> be compared is everything except the senses, and there the
differences are substantial and well
documented: salinity tolerance, depth
and zonation, body size, moult timing, tolerance of emersion and hypoxia.
Subadult Dungeness use the littoral zone in ways that matter for any comparison
drawn from trap data, red rock crab
emersion physiology has been measured in
situ, settlement and emigration
behaviour has been studied in green crab,
and predatory capability has been compared directly between green crab and red
rock crab on a native clam.</p>

<aside class="ui-source" id="ref-young2019">
  <a class="ui-source__link" href="https://doi.org/10.3390/fishes5010004" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Life History and Population Dynamics of Green Crabs (Carcinus maenas)</span>
      <span class="ui-source__meta">
        Young et al.
        · 2019 · Fishes
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-holsman2006">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps308183" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Intertidal migration and habitat use by subadult Dungeness crab Cancer magister in a NE Pacific estuary</span>
      <span class="ui-source__meta">
        Holsman et al.
        · 2006 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-defur1983">
  <a class="ui-source__link" href="https://doi.org/10.2307/1541467" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">ANALYSIS OF HEMOLYMPH OXYGEN LEVELS AND ACID-BASE STATUS DURING EMERSION 'IN SITU' IN THE RED ROCK CRAB, CANCER PRODUCTUS</span>
      <span class="ui-source__meta">
        DEFUR et al.
        · 1983 · The Biological Bulletin
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-moksnes2003">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps250215" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Settlement behavior in shore crabs Carcinus maenas: why do postlarvae emigrate from nursery habitats?</span>
      <span class="ui-source__meta">
        Moksnes et al.
        · 2003 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-nicol2025">
  <a class="ui-source__link" href="https://doi.org/10.1111/maec.70071" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Comparison of Predatory Capabilities of Invasive European Green Crabs ( Carcinus maenas ) and Native Red Rock Crabs ( Cancer productus ) Preying Upon a Common Native Bivalve ( Leukoma staminea )</span>
      <span class="ui-source__meta">
        Nicol et al.
        · 2025 · Marine Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>That list is the beginning of routes 11 and 12.</strong> Selectivity does not have to
come from the signal. It can come from the calendar.</p>

<hr />

<h2 id="predators-and-parasites">Predators and parasites</h2>

<p><strong>The complete answer to “why not biological control” is one paper.</strong> The
host specificity of <em>Sacculina carcini</em>, the parasitic barnacle proposed as a
green crab agent, has been tested against native Pacific
crabs, and the result is why nobody
deploys it. I am not going to characterise the numbers here — I hold it at
abstract level — but the conclusion is not controversial and it is the standing
reason route 9 is closed.</p>

<aside class="ui-source" id="ref-goddard2005">
  <a class="ui-source__link" href="https://doi.org/10.1007/s10530-003-2981-0" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Host specificity of Sacculina carcini, a potential biological control agent of the introduced European green crab Carcinus maenas in California</span>
      <span class="ui-source__meta">
        Goddard et al.
        · 2005 · Biological Invasions
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Route 10 has the only landscape-scale evidence in this entire review</strong>, and it
is not usable. A recovering sea otter population shows a strong negative
space-and-time relationship with green crab, with crabs persisting highest where
tidal restriction excluded the otters.
That is the best result anywhere in the predator literature — and <strong>the southern
sea otter has been absent from the Salish Sea since 1915.</strong> It is an argument
for removing tidal barriers, not a lever anyone can pull.</p>

<aside class="ui-source" id="ref-jeppesen2024">
  <a class="ui-source__link" href="https://doi.org/10.1007/s10530-024-03467-3" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Recovering population of the southern sea otter suppresses a global marine invader</span>
      <span class="ui-source__meta">
        Jeppesen et al.
        · 2024 · Biological Invasions
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>So I built a register of everything else that might eat a green crab in British
Columbia: <strong>24 agents, each carrying a status so the empty rows stay visible.</strong>
The tally is the finding — <strong>1 demonstrated, 1 failed, 3 with a measured diet
record, 4 plausible-untested, and 15 with no data at all.</strong> Five of the top six
candidates are present in the Salish Sea. <strong>None of the five has demonstrated
evidence there.</strong></p>

<p>Four survive three filters at once — present where the crabs are, capable of
taking one, and attached to a step someone could take this year: <strong>giant Pacific
octopus, marine-foraging river otter, Pacific staghorn sculpin, and the
sunflower sea star.</strong></p>

<p>Building out their biology reordered them, and the reordering is the point.
Ranked on <strong>being present and cheaply samplable</strong>, the river otter comes first.
Ranked on <strong>how strong the dietary prior actually is</strong>, the octopus does. Those
are different questions and collapsing them into one ranking is how a project
talks itself into the wrong survey. The sunflower sea star has the <strong>strongest
structural case on the list</strong> — a recovering predator with funded recovery
programmes already running for their own reasons — and the <strong>weakest dietary
case</strong>, because its entire measured feeding ecology is urchins and molluscs.
Both statements are true at once.</p>

<p><strong>What I can state, because these are my own search results rather than
somebody’s findings:</strong> no green-crab record exists in the diet literature for
<em>any</em> octopus species; there is no green-crab diet fraction for river otter
anywhere; there is nothing published on Pacific Northwest fish predation on
green crab; and I located <strong>no crustacean predation record at all</strong> for the
sunflower sea star. The diet numbers behind the ranking sit in the working notes
at abstract level, where they belong.</p>

<p><strong>And none of the four is measured on the size class that matters.</strong> Which
brings up the thing that kept recurring.</p>

<hr />

<h2 id="the-two-that-survive">The two that survive</h2>

<p><strong>Route 11 — gear.</strong> Trap entrance modification has the largest demonstrated
effect of anything in this exercise.
It is a cable tie and a sinker. Nothing the sensory workstream produced comes
close.</p>

<aside class="ui-source" id="ref-bergshoeff2018">
  <a class="ui-source__link" href="https://doi.org/10.7717/peerj.4223" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Using underwater video to evaluate the performance of the Fukui trap as a mitigation tool for the invasive European green crab ( Carcinus maenas ) in Newfoundland, Canada</span>
      <span class="ui-source__meta">
        Bergshoeff et al.
        · 2018 · PeerJ
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-bergshoeff2019">
  <a class="ui-source__link" href="https://doi.org/10.7717/peerj.6308" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Improving the efficiency of the Fukui trap as a capture tool for the invasive European green crab ( Carcinus maenas ) in Newfoundland, Canada</span>
      <span class="ui-source__meta">
        Bergshoeff et al.
        · 2019 · PeerJ
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>There is also a peer-reviewed integrated population model for this species with
public code, fitted on a multi-year
removal time series — <strong>which I confidently declared did not exist</strong>, and which
puts shrimp traps well above the trap type used throughout British Columbia on
per-trap efficiency. I would not quote a single multiplier from it: the
estimate shifts noticeably depending on which auxiliary dataset the model is
fitted with, which the authors report themselves. <strong>The defensible statement
is that a paired deployment — the two trap types fished side by side, same
days, same sites, same soak — would pin the number down cheaply with existing
gear.</strong></p>

<aside class="ui-source" id="ref-keller2025">
  <a class="ui-source__link" href="https://doi.org/10.1111/1365-2656.70176" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">An integrated integral projection model ( IPM 2 ) to disentangle size‐structured harvest and natural mortality</span>
      <span class="ui-source__meta">
        Keller et al.
        · 2025 · Journal of Animal Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p><strong>Route 12 — place and schedule.</strong> Selectivity from the calendar rather than
from a device. Two axes came out strong: <strong>trap the structured habitat rather
than the open flat</strong>, and <strong>fish the daytime flood tide</strong>, because green crab
move up-shore on the flood regardless of light while the Dungeness incursion is
nocturnal. Others came out weaker, and the axis most often cited — tidal height
alone — was <strong>downgraded</strong> by a paper showing subadult Dungeness use the
littoral zone too.</p>

<aside class="ui-source" id="ref-holsman2006">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps308183" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Intertidal migration and habitat use by subadult Dungeness crab Cancer magister in a NE Pacific estuary</span>
      <span class="ui-source__meta">
        Holsman et al.
        · 2006 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>It costs nothing, because every axis is a decision about where and when to set
gear already in the water. It is falsifiable now, at a few hundred trap-sets,
with the kill condition written in advance.</p>

<p><strong>And here is the case against it, stated as strongly as I can.</strong> It is bycatch
reduction, not control. The demographic work says only heavy size-selected
removal of <em>juveniles</em> drives the population down; composition does not. <strong>And
the gear cannot execute that lever.</strong> The smallest crab in one dataset of 17,615
animals was 21.1 mm across the carapace. Settling juveniles are 1.5 mm. <strong>The
decisive size class and the available gear are mismatched, and no amount of
siting fixes it.</strong></p>

<p>That mismatch is also true of every predator in the register. <strong>The size class
that decides the outcome is unmeasured for gear and for predators alike.</strong> If
one sentence from this whole exercise is worth carrying forward, it is that one.</p>

<hr />

<h2 id="things-that-kept-being-true">Things that kept being true</h2>

<ul>
  <li><strong>Physics beats biology at range, every time.</strong> Six of the twelve closures
came from arithmetic done before any literature search — near-field falloff,
waveguide cutoff, displacement-versus-pressure, ohmic heating. <strong>Doing the
arithmetic first would have saved weeks</strong>, and the one branch where I built
the apparatus before computing the gate is the branch that wasted the most
time.</li>
  <li><strong>A cue that works is usually a cue everyone can hear.</strong> Selectivity and
efficacy pulled against each other in every sensory route. The channel with
the best range was the least selective; the most selective idea was the one
that would not propagate.</li>
  <li><strong>Absence of a measurement is not absence of the thing.</strong> Repeatedly the
honest output was <em>unavailable</em> rather than <em>absent</em> — a prey-sound corpus
filtered before the relevant band, native species never tested, a receptor
never sought. Collapsing those into a null manufactures a confident negative
out of a test nobody ran.</li>
  <li><strong>The literature on the invader is far better than the literature on the
natives.</strong> Green crab is a laboratory animal. The commercially important
Pacific crabs it competes with are not, and every cross-species comparison in
this review foundered on that asymmetry rather than on modelling.</li>
  <li><strong>Removal suppresses locally and does not
extirpate</strong>. That is the consistent
finding across jurisdictions, including a documented case of
<strong>stage-specific overcompensation — the hydra effect — following adult-only
removal</strong>, whose possibility had been
assessed in advance.
Early detection has a much better record.</li>
  <li><strong>The temperature literature is where the actual predictive signal is.</strong>
Adult thermal tolerance does not discriminate sites — it is broad enough to
make the whole coast suitable. The
discriminator is larval recruitment
temperature, with warmer winters
adding a second brood and a modelling
result finding a large increase in larval arrival for a small temperature
rise. The adaptive-genomics literature for
this species is likewise about
temperature,
not about reproduction or sensory biology — an observation about what the
literature is <em>about</em>, which is a claim I can make from titles and abstracts.</li>
</ul>

<aside class="ui-source" id="ref-ens2022">
  <a class="ui-source__link" href="https://doi.org/10.1139/er-2021-0059" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">The Green Wave: reviewing the environmental impacts of the invasive European green crab ( Carcinus maenas ) and potential management approaches</span>
      <span class="ui-source__meta">
        Ens et al.
        · 2022 · Environmental Reviews
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-grosholz2021">
  <a class="ui-source__link" href="https://doi.org/10.1073/pnas.2003955118" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Stage-specific overcompensation, the hydra effect, and the failure to eradicate an invasive predator</span>
      <span class="ui-source__meta">
        Grosholz et al.
        · 2021 · Proceedings of the National Academy of Sciences
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-turner2015">
  <a class="ui-source__link" href="https://doi.org/10.1007/s10530-015-1026-9" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Assessing population increase as a possible outcome to management of invasive species</span>
      <span class="ui-source__meta">
        Turner et al.
        · 2015 · Biological Invasions
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-grason2018">
  <a class="ui-source__link" href="https://doi.org/10.3391/mbi.2018.9.1.04" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Citizen science program detects range expansion of the globally invasive European green crab in Washington State (USA)</span>
      <span class="ui-source__meta">
        Grason et al.
        · 2018 · Management of Biological Invasions
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-compton2010">
  <a class="ui-source__link" href="https://doi.org/10.1111/j.1472-4642.2010.00644.x" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Thermogeography predicts the potential global range of the invasive European green crab (Carcinus maenas)</span>
      <span class="ui-source__meta">
        Compton et al.
        · 2010 · Diversity and Distributions
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-derivera2006">
  <a class="ui-source__link" href="https://doi.org/10.1007/s00227-006-0451-9" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Larval development rate predicts range expansion of an introduced crab</span>
      <span class="ui-source__meta">
        deRivera et al.
        · 2006 · Marine Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-rey2017">
  <a class="ui-source__link" href="https://doi.org/10.1007/s12237-017-0235-0" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Effect of Maternal Size, Reproductive Season and Interannual Variability in Offspring Provisioning of Carcinus maenas in a Coastal Lagoon</span>
      <span class="ui-source__meta">
        Rey et al.
        · 2017 · Estuaries and Coasts
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-du2024">
  <a class="ui-source__link" href="https://doi.org/10.1016/j.pocean.2024.103245" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Dispersal pathways of European green crab larvae into and throughout the eastern Salish Sea</span>
      <span class="ui-source__meta">
        Du et al.
        · 2024 · Progress in Oceanography
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-tepolt2020">
  <a class="ui-source__link" href="https://doi.org/10.3389/fevo.2020.580701" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Rapid Adaptation to Temperature via a Potential Genomic Island of Divergence in the Invasive Green Crab, Carcinus maenas</span>
      <span class="ui-source__meta">
        Tepolt et al.
        · 2020 · Frontiers in Ecology and Evolution
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-thia2021">
  <a class="ui-source__link" href="https://doi.org/10.1111/mec.16258" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Ready on arrival: Standing variation at a chromosomal inversion contributes to rapid adaptation in an invasive marine crab</span>
      <span class="ui-source__meta">
        Thia
        · 2021 · Molecular Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-venkataraman2025">
  <a class="ui-source__link" href="https://doi.org/10.1101/2025.04.22.650023" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Plasticity, not genetics, shapes individual responses to thermal stress in non-native populations of the European green crab ( Carcinus maenas )</span>
      <span class="ui-source__meta">
        Venkataraman et al.
        · 2025
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<hr />

<h2 id="the-method-and-the-errors-it-caught">The method, and the errors it caught</h2>

<p>The part of this I would actually defend is not any of the twelve verdicts. It
is that <strong>every constant is pinned by a test that fails if the figure is
misquoted</strong>, every number carries a tag saying whether it was measured, derived,
assumed or unavailable, and <strong>a source read only at abstract may be cited as
existing but may not have findings attributed to it.</strong></p>

<p>That last rule is unpopular with my own drafts. It caught five violations in the
first version of the companion post, and it is why several paragraphs above name
what a study measured rather than what it found.</p>

<p><strong>Here is what those rules caught. I think this table is the most useful thing
on the page.</strong></p>

<table>
  <thead>
    <tr>
      <th>The error</th>
      <th>How it was caught</th>
      <th>What it cost</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td>A turbulent-diffusion constant <strong>10× wrong</strong></td>
      <td>Checked against a field measurement</td>
      <td>Chemical detection range was off by an order of magnitude in the <em>conservative</em> direction</td>
    </tr>
    <tr>
      <td>Scored far-field stimuli against a <strong>tactile</strong> receptor</td>
      <td>Reading the paper properly</td>
      <td>Invalidated a whole class of range estimates</td>
    </tr>
    <tr>
      <td>Attributed a vibration organ to the <strong>wrong joint</strong>, then used a surrogate band from the wrong genus</td>
      <td>Re-reading the 1954 source</td>
      <td>Reversed a result: “1 of 9 prey sounds rescued” became <strong>0 of 9</strong></td>
    </tr>
    <tr>
      <td>Conflated a trap’s <strong>entry success</strong> with its <strong>catch increase</strong></td>
      <td>A test asserting the two figures</td>
      <td>The best modification is +81%, not the number I had</td>
    </tr>
    <tr>
      <td>Collapsed a lab mechanism into a <strong>population-level</strong> claim</td>
      <td>The operator asked what a phrase meant</td>
      <td>Split into two claims; pinned that no population-level effect has been demonstrated</td>
    </tr>
    <tr>
      <td>“<strong>Zero</strong> native sensory channels have ever been measured”</td>
      <td>Searching again, less shallowly</td>
      <td>A strong negative from a shallow search. Overturned within minutes</td>
    </tr>
    <tr>
      <td>“<strong>No population model exists</strong> for this species”</td>
      <td>Searching by <em>author</em> instead of by topic</td>
      <td>It existed, with public code. The repos are named after the method, not the species</td>
    </tr>
    <tr>
      <td>Read a gear ratio <strong>off a log axis by eye</strong></td>
      <td>Reading the printed posterior table</td>
      <td>Both comparison gears understated, <strong>always in the direction that flattered my preferred answer</strong></td>
    </tr>
  </tbody>
</table>

<aside class="ui-source" id="ref-mcdonald2001">
  <a class="ui-source__link" href="https://doi.org/10.1016/S0022-0981(00)00344-0" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">The competitive and predatory impacts of the nonindigenous crab Carcinus maenas (L.) on early benthic phase Dungeness crab Cancer magister Dana</span>
      <span class="ui-source__meta">
        McDonald et al.
        · 2001 · Journal of Experimental Marine Biology and Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Two patterns in that table are worth more than the individual entries.</strong></p>

<p>The first: <strong>most of these errors ran in the direction that made the result
look better.</strong> Not one of them was random. That is what a bias looks like from
the inside, and it is the argument for tests that pin numbers rather than
vigilance.</p>

<p>The second: <strong>a test can hold a wrong number in place.</strong> The “zero native
channels” claim survived two days after I knew it was wrong, because a test was
asserting it, with a comment beside it saying the value was known to be stale.
That is worse than an unchecked number — it looks checked. And when I finally
corrected it, the fix nearly introduced a new error: the function answering
<em>which channels are comparable across species</em> tested only whether a cell was
marked “measured”, so filling the two Dungeness cells would have certified a
category error as a comparison. <strong>A check that counts statuses will happily
certify nonsense.</strong></p>

<hr />

<h2 id="what-would-change-the-picture">What would change the picture</h2>

<ul>
  <li><strong>A thermocouple in a Helmholtz coil tank</strong>, during a replication with a sham
coil. Settles route 2 either way, and it is the cheapest decisive experiment
in the review.</li>
  <li><strong>A measured audiogram for green crab, Dungeness and red rock crab on one
rig.</strong> It does not exist. It is the single measurement that would change the
most, and if the bands turned out to differ substantially, most of the
mechanical conclusions above would need redoing.</li>
  <li><strong>A paired deployment of two trap types</strong>, same days and sites. Settles the
gear question with equipment already in the water.</li>
  <li><strong>Any diet study at all</strong> on the four shortlisted predators — two of which
need no collection permit, because middens and scat are lying on the ground.</li>
  <li><strong>Gear that reaches sub-20 mm crabs.</strong> Nothing in this review addresses the
size class that the demography says decides the outcome. That is the open
problem, and I do not have an answer to it.</li>
</ul>

<p>If any of this is useful to somebody working on a real protocol, it is yours —
that is why it is here rather than in a private folder. The working notes,
including the numbers I have held back above because I have only read their
abstracts, are more detailed than this post and I am happy to share them.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[A screening exercise across sensory, biological and operational mechanisms for controlling an invasive crab — what each route would need to be true, what closed it, and the two that are still standing.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/european-green-crab.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/european-green-crab.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">A research assistant that keeps nothing</title><link href="https://polarize.tech/blog/a-research-assistant-that-keeps-nothing/" rel="alternate" type="text/html" title="A research assistant that keeps nothing" /><published>2026-09-15T07:00:00-06:00</published><updated>2026-09-15T07:00:00-06:00</updated><id>https://polarize.tech/blog/a-research-assistant-that-keeps-nothing</id><content type="html" xml:base="https://polarize.tech/blog/a-research-assistant-that-keeps-nothing/"><![CDATA[<p>A tool write-up. zdr-research-chat is the research assistant behind this site: a chat and
voice interface to a language model where every component that touches the conversation runs
on the author’s own machine. Built for work that produces a written record.</p>

<h2 id="what-runs-where">What runs where</h2>

<table>
  <thead>
    <tr>
      <th>function</th>
      <th>runs on</th>
      <th>leaves the machine</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td>language model</td>
      <td>Ollama, host-native, on the GPU</td>
      <td>no</td>
    </tr>
    <tr>
      <td>embeddings</td>
      <td>Ollama, host-native</td>
      <td>no</td>
    </tr>
    <tr>
      <td>chat interface and retrieval</td>
      <td>Open WebUI, in a container</td>
      <td>no</td>
    </tr>
    <tr>
      <td>vector store</td>
      <td>Qdrant, in a container</td>
      <td>no</td>
    </tr>
    <tr>
      <td>speech-to-text</td>
      <td>faster-whisper, inside Open WebUI</td>
      <td>no</td>
    </tr>
    <tr>
      <td>text-to-speech</td>
      <td>Kokoro, host-native</td>
      <td>no</td>
    </tr>
    <tr>
      <td>phone access</td>
      <td>Tailscale private network, HTTPS</td>
      <td>encrypted end to end between own devices</td>
    </tr>
    <tr>
      <td>journal</td>
      <td>a local git repository</td>
      <td>only on push, to its own private remote</td>
    </tr>
  </tbody>
</table>

<p>The model and the voice synthesis run outside containers because containers on Apple Silicon
cannot reach the GPU. Everything else is in containers and bound to loopback.</p>

<h2 id="checking-the-claim">Checking the claim</h2>

<p>Zero retention is stated as something to verify, not something to trust. Three checks:</p>

<ol>
  <li><strong>List live connections during a conversation.</strong> Nothing in the chat path should connect
anywhere but the local machine.</li>
  <li><strong>Turn off Wi-Fi.</strong> Chat, retrieval, speech-to-text and text-to-speech keep working. Only
phone access and journal pushes need a network.</li>
  <li><strong>Read the switches.</strong> Open WebUI’s telemetry, analytics, update check and web search are
off in the environment file. Qdrant’s usage statistics are off in the compose file.</li>
</ol>

<p><strong>The Qdrant switch was missing until 2026-09-15.</strong> Qdrant ships with usage statistics on,
and the stack never turned them off, so one of its two containers was sending anonymised
usage data while the documentation said telemetry was off. Found while checking this write-up
against the code rather than the README. The switch is now set, and the repository’s
self-check fails if it is ever removed.</p>

<h2 id="where-it-deliberately-is-not-zero-retention">Where it deliberately is not zero-retention</h2>

<p>Four exceptions, each off unless switched on, each documented in the file that makes the
request.</p>

<table>
  <thead>
    <tr>
      <th>tool</th>
      <th>reaches</th>
      <th>sends</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td>literature search</td>
      <td>OpenAlex, Europe PMC, Crossref, DANDI</td>
      <td>search terms and DOIs</td>
    </tr>
    <tr>
      <td>web search</td>
      <td>DuckDuckGo</td>
      <td>the query; disabled in the shipped config, and per chat when enabled</td>
    </tr>
    <tr>
      <td>air quality</td>
      <td>OpenAQ, and a geocoder if given a place name</td>
      <td>coordinates or the place name</td>
    </tr>
    <tr>
      <td>video transcripts</td>
      <td>YouTube</td>
      <td>a public video id</td>
    </tr>
  </tbody>
</table>

<p>None of these sees the conversation. A search query is still data, and those services log
requests like any website.</p>

<h2 id="a-tier-not-a-slogan">A tier, not a slogan</h2>

<p>“Zero data retention” describes where the stack is pointed, not the code. Every model,
embedding, speech and voice backend is a URL. The deployment declares which tier it is in:</p>

<table>
  <thead>
    <tr>
      <th>tier</th>
      <th>means</th>
      <th>checkable how</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td>local</td>
      <td>every backend on this machine</td>
      <td>a connection listing during a conversation</td>
    </tr>
    <tr>
      <td>self-hosted</td>
      <td>own hardware, own jurisdiction</td>
      <td>own network</td>
    </tr>
    <tr>
      <td>managed zero-retention</td>
      <td>a vendor with a contractual guarantee</td>
      <td>not checkable — a contract, not a measurement</td>
    </tr>
    <tr>
      <td>cloud</td>
      <td>no guarantee</td>
      <td>—</td>
    </tr>
  </tbody>
</table>

<p>Only <code class="language-plaintext highlighter-rouge">local</code> can be verified from the machine itself. It is the default.</p>

<h2 id="the-journal">The journal</h2>

<p>The assistant can make three kinds of write — a finding, a theory update, a session log —
into a separate git repository.</p>

<ul>
  <li><strong>Only on an explicit request</strong> (“log that”, “save this”). Otherwise the write is refused
and the assistant says nothing was written.</li>
  <li><strong>One commit per write, append-only.</strong> No amend, no rebase, no force-push, no whole-file
rewrite. The history of a theory file is the history of the thinking.</li>
  <li><strong>The container never runs git.</strong> The tool writes the file and queues a request; a
committer on the host turns each request into one commit. A crashed container cannot leave
a repository half-written.</li>
</ul>

<h2 id="literature-the-model-only-asks">Literature: the model only asks</h2>

<p>In the literature tool the model’s whole job is to turn a request into search terms and pick
a function. The archive ranks the results. The tool draws titles, authors, abstracts and
retraction notices straight from the archive’s records into a panel. The model is told the
reader can already see the panel and not to restate it.</p>

<p><strong>A citation on screen never passed through the model</strong>, so the model cannot misquote it.
Tools that place a language model between the reader and the paper are deliberately not
used. The archives are a fixed allowlist of four hosts, enforced in code.</p>

<h2 id="memory-is-the-design-constraint">Memory is the design constraint</h2>

<p>On a 16 GB machine the model shares memory with the containers, the embedding model and the
operating system. If the machine is swapping, the model is too big, and no quantisation
setting recovers it. A smaller model that fits in memory beats a larger one that pages.</p>

<p>Two further rules from running it:</p>

<ul>
  <li><strong>Avoid models that reason before calling a tool.</strong> Journal writes and searches are tool
calls; a model that thinks at length before each one turns a voice exchange into a wait.</li>
  <li><strong>Raise the context length.</strong> The runtime’s default context is small enough that a system
prompt plus a few tool definitions can silently push the tools out.</li>
</ul>

<h2 id="why-a-firewall-ships-with-it">Why a firewall ships with it</h2>

<p>A laptop can hold a publicly routable address with no router in front of it. Then every
service listening on all interfaces is on the open internet — including a model server that
must listen beyond loopback so the containers can reach it.</p>

<p>On the machine this was built on, that was not hypothetical. Counted from the model server’s
own access log: <strong>1,009 successful inference requests from 160 addresses outside any private
or tailnet range</strong>, 5,985 outside requests in all, between 15 August and 9 September 2026.
The last is on 9 September, the day a default-deny firewall for the public interface was
committed. Local requests continue in the same log after it.</p>

<p>So the firewall travels with the stack: loopback, the tailnet and the container bridge stay
open, the public interface does not. A network check reports in one line whether a newly
joined network is hiding the machine or exposing it.</p>

<h2 id="limits">Limits</h2>

<ul>
  <li><strong>An 8B-class model on a laptop is not a frontier model.</strong> The trade is capability for
being usable with material that should not be uploaded.</li>
  <li><strong>macOS on Apple Silicon only</strong>, 16 GB minimum. The GPU paths assume it.</li>
  <li><strong>Tailscale’s coordination service sees device metadata</strong>, not content.</li>
  <li><strong>The four exceptions above are real egress</strong> whenever they are switched on.</li>
</ul>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[zdr-research-chat: a voice research assistant where the model, embeddings, speech-to-text and text-to-speech all run on one machine — how the zero-retention claim is checked, and the four places it deliberately is not true.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/locked-laptop.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/locked-laptop.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">A hive and a cortex, described the same way</title><link href="https://polarize.tech/blog/a-hive-and-a-cortex-described-the-same-way/" rel="alternate" type="text/html" title="A hive and a cortex, described the same way" /><published>2026-09-12T07:00:00-06:00</published><updated>2026-09-12T07:00:00-06:00</updated><id>https://polarize.tech/blog/a-hive-and-a-cortex-described-the-same-way</id><content type="html" xml:base="https://polarize.tech/blog/a-hive-and-a-cortex-described-the-same-way/"><![CDATA[<p>An inventory. The parallel below is not mine and is not new.</p>

<h2 id="the-parallel-and-whose-it-is">The parallel, and whose it is</h2>

<p>A swarm choosing between two nest sites and a cortical population choosing which way dots
move have been given one formal description.</p>

<aside class="ui-source" id="ref-marshall2009b">
  <a class="ui-source__link" href="https://doi.org/10.1098/rsif.2008.0511" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">On optimal decision-making in brains and social insect colonies</span>
      <span class="ui-source__meta">
        Marshall et al.
        · 2009 · Journal of The Royal Society Interface
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a><p class="ui-source__note">The formal treatment. Read at full text for the sections carrying its conclusions; the model derivations were not read.</p>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>That paper dates the idea to “at least Hofstadter (1979)” in its own introduction, and
describes itself as a first step toward a common framework — one built on how a system’s
components interact rather than on what they are.</p>

<aside class="ui-source" id="ref-marshall2009">
  <a class="ui-source__link" href="https://doi.org/10.1016/j.cub.2009.03.011" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Colony-level cognition</span>
      <span class="ui-source__meta">
        Marshall et al.
        · 2009 · Current Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a><p class="ui-source__note">Same authors, same year, the idea under a different heading.</p>
</aside>

<p>The experimental work usually paired with it concerns inhibitory signalling between scouts.
Its title and framing put the comparison to brains in front, rather than leaving it to a
reader.</p>

<aside class="ui-source" id="ref-seeley2012">
  <a class="ui-source__link" href="https://doi.org/10.1126/science.1210361" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Stop Signals Provide Cross Inhibition in Collective Decision-Making by Honeybee Swarms</span>
      <span class="ui-source__meta">
        Seeley et al.
        · 2012 · Science
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a><p class="ui-source__note">The experimental result usually paired with the framework above.</p>
</aside>

<h2 id="what-the-description-covers">What the description covers</h2>

<p>Three properties, per the 2009 treatment:</p>

<ul>
  <li><strong>Populations, not individuals.</strong> Interacting populations accumulate noisy evidence for
competing alternatives.</li>
  <li><strong>A threshold on one population.</strong> The alternative whose population crosses first is the
one taken.</li>
  <li><strong>A threshold that moves.</strong> Raising it buys accuracy and costs speed. A parameter in the
cortical model; a headcount at a site in the ants.</li>
</ul>

<p>The claim is stronger than resemblance. Under particular settings the cortical model
reduces to a diffusion process implementing the sequential probability ratio test — for a
two-way choice, the procedure minimising decision time at any given error rate. The
analysis asks which colony models do the same, and treats the answer as a prediction about
how colonies should behave if deciding optimally.</p>

<p>Past two options the analysis changes.</p>

<aside class="ui-source" id="ref-reina2017">
  <a class="ui-source__link" href="https://doi.org/10.1103/physreve.95.052411" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Model of the best-of-Nnest-site selection process in honeybees</span>
      <span class="ui-source__meta">
        Reina et al.
        · 2017 · Physical Review E
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a><p class="ui-source__note">Extends the analysis past two options.</p>
</aside>

<p>This is also where the literature meets the best-of-N problem in distributed and robotic
systems — the same problem stated without the bees.</p>

<h2 id="where-its-own-authors-say-it-stops">Where its own authors say it stops</h2>

<p><strong>The colony must go and get its evidence.</strong> In the cortical task, evidence for both
alternatives arrives at a fixed equal rate. Scouts discover sites stochastically, leaving
an explore-or-exploit problem the cortical version does not have: assess what is known, or
look for better. The authors call it a hybrid of a bandit problem and a
minimum-decision-time problem, and say nobody had formalised it.</p>

<p><strong>Consensus is not foraging.</strong> The paper states that colony emigration is <em>optimal
consensus</em> decision-making and “differs from the problem of distributed resource intake
maximization that colonies tackle during foraging.” Quorum figures and the cross-inhibition
result come from nest-site selection during swarming. Foraging recruitment runs on
different machinery. A description that moves between the two is describing two systems.</p>

<h2 id="two-extensions-neither-established">Two extensions, neither established</h2>

<p>Recorded as framings, not findings.</p>

<p><strong>A modulatory layer.</strong> The models have recruitment and inhibition, and nothing setting the
regime those run in. Bees have candidates.</p>

<aside class="ui-source" id="ref-barron2007">
  <a class="ui-source__link" href="https://doi.org/10.1073/pnas.0610506104" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Octopamine modulates honey bee dance behavior</span>
      <span class="ui-source__meta">
        Barron et al.
        · 2007 · Proceedings of the National Academy of Sciences
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-linn2020">
  <a class="ui-source__link" href="https://doi.org/10.1098/rspb.2020.1950" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Octopamine and dopamine mediate waggle dance following and information use in honeybees</span>
      <span class="ui-source__meta">
        Linn et al.
        · 2020 · Proceedings of the Royal Society B: Biological Sciences
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-dong2023">
  <a class="ui-source__link" href="https://doi.org/10.1016/j.cub.2023.03.072" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">An inhibitory signal associated with danger reduces honeybee dopamine levels</span>
      <span class="ui-source__meta">
        Dong et al.
        · 2023 · Current Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>Whether these belong in the architecture as a separate axis — gain rather than content — is
untested. The third cuts across the tidy version: if a targeted inhibitory signal moves a
diffuse modulator, then selecting among candidates and setting the regime are not cleanly
separable.</p>

<p><strong>A write step.</strong> Queen pheromone has been examined against expression of genes responsible
for epigenetic modifications in worker brains.</p>

<aside class="ui-source" id="ref-cardosojunior2020">
  <a class="ui-source__link" href="https://doi.org/10.1098/rsbl.2020.0440" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Queen pheromone modulates the expression of epigenetic modifier genes in the brain of honeybee workers</span>
      <span class="ui-source__meta">
        Cardoso-Junior et al.
        · 2020 · Biology Letters
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>Placing that as the durable-change step is an analogy across levels. The level mismatch is
real: the bee side is role-level — dancer, follower, scout — and the neural side is
cell-type-level.</p>

<h2 id="two-observations-that-cut-the-other-way">Two observations that cut the other way</h2>

<p><strong>The signal is shaped by its audience.</strong> Removing bees from the dance floor, and separately
replacing adults with bees too young to follow, was used to test whether dance information
content depends on who is watching. Directional and distance precision tracked follower
numbers; mean waggle-run duration and distance per run are reported unchanged.</p>

<aside class="ui-source" id="ref-lin2026">
  <a class="ui-source__link" href="https://doi.org/10.1073/pnas.2518687123" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">The audience shapes the information content of the honey bee waggle dance</span>
      <span class="ui-source__meta">
        Lin et al.
        · 2026 · Proceedings of the National Academy of Sciences
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a><p class="ui-source__note">Results section read in full. The statistics quoted here come from it; no interpretation is attributed to it.</p>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>A variance effect, not a bias effect. A population whose output precision depends on its
readership is not a one-way sender.</p>

<p><strong>No offline replay on the bee side.</strong> The dance is a waggle run, then a return loop
alternating left and right. The loop repositions; no reversed waggle run is reported.
Compressed reactivation of place-cell sequences in both directions is a large neural
literature. The bee-side absence is absence of reported evidence, not a study that looked.</p>

<aside class="ui-source" id="ref-dong2023b">
  <a class="ui-source__link" href="https://doi.org/10.1126/science.ade1702" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Social signal learning of the waggle dance in honey bees</span>
      <span class="ui-source__meta">
        Dong et al.
        · 2023 · Science
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<h2 id="what-would-make-this-wrong">What would make this wrong</h2>

<ul>
  <li>Follower recruitment determined almost entirely by instantaneous dance properties, with
no contribution from prior dance-floor state.</li>
  <li>Simultaneous dances that do not measurably interact through competition for a finite pool.</li>
  <li>Cross-inhibition in swarms and cortex producing qualitatively different dynamics under
matched conditions.</li>
  <li>Thresholds turning out to be observer cutoffs rather than nonlinear population
transitions.</li>
</ul>

<p>One caution on the neural side. Reaching for cortical disinhibition as the mechanism of
attention and then borrowing it imports an unsettled claim.</p>

<aside class="ui-source" id="ref-myersjoseph2024">
  <a class="ui-source__link" href="https://doi.org/10.1016/j.neuron.2023.11.006" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Disinhibition by VIP interneurons is orthogonal to cross-modal attentional modulation in primary visual cortex</span>
      <span class="ui-source__meta">
        Myers-Joseph et al.
        · 2024 · Neuron
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a><p class="ui-source__note">Published version of a preprint; the published title narrows the claim to cross-modal attention.</p>
</aside>

<h2 id="on-sources">On sources</h2>

<p>Two of the papers above were read beyond their abstracts: the 2009 framework, in the
sections carrying its conclusions, and the audience study, its results section. The rest are
entry points. Where this post says a study <em>examined</em> or <em>tested</em> something, that wording is
load-bearing — it marks pointing at a result rather than having checked it.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[A honeybee colony choosing a nest and a cortical population choosing between two motions have carried the same formal description since 2009. What it covers, and where its own authors say it stops.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/waggle-dance.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/waggle-dance.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">Building a sensory screening tool for the European green crab</title><link href="https://polarize.tech/blog/green-crab-sensory-screening-tool/" rel="alternate" type="text/html" title="Building a sensory screening tool for the European green crab" /><published>2026-09-06T09:00:00-06:00</published><updated>2026-09-06T09:00:00-06:00</updated><id>https://polarize.tech/blog/green-crab-sensory-screening-tool</id><content type="html" xml:base="https://polarize.tech/blog/green-crab-sensory-screening-tool/"><![CDATA[<p>The European green crab (<em>Carcinus maenas</em>) is unusual among invasive species in being a
classic laboratory animal. That makes it a test of a question worth asking about any
organism: <strong>how much of its sensory front end can be computed rather than assumed?</strong></p>

<p>Not a simulator. A simulator implies you turn a crank and get behaviour out. This is
narrower: for a given stimulus it answers <strong>how much</strong> arrives at a receptor, <strong>in what
format</strong> that receptor passes it on, and <strong>where</strong> it goes — and refuses when the number
underneath does not exist. The most common output is a refusal.</p>

<h2 id="the-design-rule">The design rule</h2>

<p>Every constant carries its provenance: measured in this species, measured in a surrogate,
derived from physics, or assumed. That sounds like bookkeeping. It did the work.</p>

<p>The tags caught six errors already in the model, every one from reading a summary instead of
a source. Two examples:</p>

<ul>
  <li>A trap statistic entered as “entry success rises from 16% to 59%.” Those are two different
measurements — one the fraction of attempts that succeed, the other a percentage <em>increase
in catch</em> from a modification. The second does not continue the first, and the best
modification was not the one being quoted.</li>
</ul>

<aside class="ui-source" id="ref-bergshoeff2018">
  <a class="ui-source__link" href="https://doi.org/10.7717/peerj.4223" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Using underwater video to evaluate the performance of the Fukui trap as a mitigation tool for the invasive European green crab ( Carcinus maenas ) in Newfoundland, Canada</span>
      <span class="ui-source__meta">
        Bergshoeff et al.
        · 2018 · PeerJ
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-bergshoeff2019">
  <a class="ui-source__link" href="https://doi.org/10.7717/peerj.6308" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Improving the efficiency of the Fukui trap as a capture tool for the invasive European green crab ( Carcinus maenas ) in Newfoundland, Canada</span>
      <span class="ui-source__meta">
        Bergshoeff et al.
        · 2019 · PeerJ
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<ul>
  <li>A receptor threshold was carried as a single value where the study reports a range. The
single number was the low end.</li>
</ul>

<p><strong>The rule that generates the rest: an abstract is not a paper.</strong> A source read only at
abstract may be cited as existing; nothing may be said about what it measured. That
constraint is load-bearing below, and it is marked where it bites.</p>

<h2 id="mechanical-senses--the-measured-part">Mechanical senses — the measured part</h2>

<p>The strongest ground, because there is a real transfer function for this species. Mouthpart
setae recordings give displacement thresholds in micrometres and, more usefully, the coding:
spike count scales with displacement amplitude, interspike interval with velocity, and
roughly half the cells are directionally sensitive.</p>

<aside class="ui-source" id="ref-garm2005">
  <a class="ui-source__link" href="https://doi.org/10.1007/s00227-005-0020-7" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Mechanosensory properties of the mouthpart setae of the European shore crab Carcinus maenas</span>
      <span class="ui-source__meta">
        Garm
        · 2005 · Marine Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p><strong>That detail is what made the first version wrong.</strong> Those setae are <strong>tactile</strong> receptors
for handling prey, not distance detectors, and far-field stimuli were being scored against
them. The tool now raises a scope flag on any far-field verdict from that row.</p>

<p>The receptor that <em>is</em> for water motion is a different one — sensory hairs on the chelae,
studied in crayfish. A joint organ in the walking leg has been described in green crab
itself, the response of intact animals to substrate vibration tested directly, decapod
acoustic detection reviewed as a field, an evoked-potential study in American lobster asks
which organ is responsible, and a consolidated review of green crab sensory biology exists.</p>

<aside class="ui-source" id="ref-tautz1980">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.88.1.351" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">The Detection of Waterborne Vibration by Sensory Hairs on the Chelae of the Crayfish</span>
      <span class="ui-source__meta">
        Tautz et al.
        · 1980 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-burke1954">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.31.1.127" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">An Organ for Proprioception and Vibration Sense in Carcinus Maenas</span>
      <span class="ui-source__meta">
        Burke
        · 1954 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-aimon2021">
  <a class="ui-source__link" href="https://doi.org/10.1016/j.envpol.2021.117148" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Anthropogenic underwater vibrations are sensed and stressful for the shore crab Carcinus maenas</span>
      <span class="ui-source__meta">
        Aimon et al.
        · 2021 · Environmental Pollution
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-popper2001">
  <a class="ui-source__link" href="https://doi.org/10.1007/s003590100184" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Acoustic detection and communication by decapod crustaceans</span>
      <span class="ui-source__meta">
        Popper et al.
        · 2001 · Journal of Comparative Physiology A: Sensory, Neural, and Behavioral Physiology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-jzquel2021">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.240747" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Sound detection by the American lobster (Homarus americanus)</span>
      <span class="ui-source__meta">
        Jézéquel et al.
        · 2021 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-jury2024">
  <a class="ui-source__link" href="https://doi.org/10.1016/B978-0-323-99694-5.00004-0" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Sensory biology and behaviour</span>
      <span class="ui-source__meta">
        Jury et al.
        · 2024 · Ecophysiology of the European Green Crab (Carcinus Maenas) and Related Species
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Where the abstract-only rule bites:</strong> of the seven sources in this section, two were read
at full text. For the other five: they exist, and the question they asked is stated, not what
they found. <strong>So the surrogate threshold the tool uses for the water-motion channel is a
number I cannot attribute</strong>, and it is tagged as a surrogate for that reason.</p>

<h2 id="the-physics-that-decides-most-of-it">The physics that decides most of it</h2>

<p><strong>Near-field falloff.</strong> A small oscillating body in water produces a field falling off as
1/r³ if it oscillates back and forth, 1/r² if it changes volume. The cube law is brutal: a
thousand times more source amplitude buys ten times the range. Ordinary prey is a
centimetre-scale cue; only a large struggling animal or another crab reaches decimetres.</p>

<p><strong>Displacement is not pressure.</strong> Particle displacement equals velocity over 2πf, so for a
given sound pressure a kilohertz signal carries far less displacement than a hundred-hertz
one. High-frequency sound is displacement-poor, and crabs detect displacement.</p>

<p>Together these explain why the acoustic route keeps failing and the chemical route keeps
winning: a plume falls off as 1/r, and the olfactory threshold is low.</p>

<h2 id="what-prey-actually-emit">What prey actually emit</h2>

<p>The reference dataset for benthic invertebrate sound gives calibrated source levels for
scallops, limpets, urchins and crustaceans.</p>

<aside class="ui-source" id="ref-coquereau2016">
  <a class="ui-source__link" href="https://doi.org/10.1007/s00227-016-2902-2" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Sound production and associated behaviours of benthic invertebrates from a coastal habitat in the north-east Atlantic</span>
      <span class="ui-source__meta">
        Coquereau et al.
        · 2016 · Marine Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>Converted to particle displacement and solved against the crab’s threshold, none reaches a
crab at more than millimetres — and every sound in that dataset peaks between 5 and 49 kHz,
while the analysis band was filtered from 2 kHz upward. <strong>The corpus was built for hydrophone
monitoring, not prey detection, and the crab’s band was removed before analysis.</strong> A null
there is unavailable, not absent.</p>

<p>The promising cue is not a sound. Porewater pressure signals from infaunal activity have been
recorded directly in sediment, and the irrigation timing of three tellinid bivalves —
including a Pacific Northwest clam that is real green crab prey — has been measured.</p>

<aside class="ui-source" id="ref-wethey2005">
  <a class="ui-source__link" href="https://doi.org/10.2307/3593131" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Infaunal Hydraulics Generate Porewater Pressure Signals</span>
      <span class="ui-source__meta">
        Wethey et al.
        · 2005 · The Biological Bulletin
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-volkenborn2012">
  <a class="ui-source__link" href="https://doi.org/10.1357/002224012806770955" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Intermittent bioirrigation and oxygen dynamics in permeable sediments: An experimental and modeling study of three tellinid bivalves</span>
      <span class="ui-source__meta">
        Volkenborn et al.
        · 2012 · Journal of Marine Research
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>A slow hydraulic signal, not an acoustic one, and the only prey cue here with a field
detection range measured on relevant species.</p>

<h2 id="chemistry-which-out-ranges-everything">Chemistry, which out-ranges everything</h2>

<p>Modelled as a plume, chemical detection spans roughly three orders of magnitude more
distance than any mechanical cue. Two anatomically separate systems do different jobs —
olfaction on the antennules, contact chemoreception on the dactyls, where the gustatory
organs of this species have been characterised electrophysiologically.</p>

<aside class="ui-source" id="ref-schmidt1989">
  <a class="ui-source__link" href="https://doi.org/10.1007/BF00193467" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Specificity and response characteristics of gustatory sensilla (funnel-canal organs) on the dactyls of the shore crab, Carcinus maenas (Crustacea, Decapoda)</span>
      <span class="ui-source__meta">
        Schmidt et al.
        · 1989 · Journal of Comparative Physiology A
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Abstract only, so the threshold separation between the two — which is what the tool runs
on — is a sourced parameter in the model and is not stated here.</strong></p>

<p>One deliberate refusal: a chemical stimulus is not a scalar. You cannot hand it a single
concentration and get a receptor response, because mixtures cross-adapt and receptors encode
a ratio against background rather than an absolute. Single-compound dose-response is enabled;
mixtures raise an exception.</p>

<p>The female sex pheromone has been identified, and later work with it produced the most
interesting behavioural result in this review.</p>

<aside class="ui-source" id="ref-hardege2011">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps09226" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Identification of a female sex pheromone in Carcinus maenas</span>
      <span class="ui-source__meta">
        Hardege et al.
        · 2011 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-rising2022">
  <a class="ui-source__link" href="https://doi.org/10.1371/journal.pone.0276889" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Anthropogenic noise may impair the mating behaviour of the Shore Crab Carcinus Maenas</span>
      <span class="ui-source__meta">
        Rising et al.
        · 2022 · PLOS ONE
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>Males presented with a pheromone-treated dummy female showed a mating response 87% of the
time under ambient conditions and 40% under ship-noise playback — while the <em>time taken to
respond to the pheromone</em> did not change significantly. <strong>Noise interfered with completing
the behaviour, not with detecting the signal.</strong> That dissociation is worth more than either
number alone.</p>

<h2 id="electric-and-magnetic--where-the-tool-says-no">Electric and magnetic — where the tool says no</h2>

<p>The two channels refused outright, and the refusals are its highest-confidence outputs.</p>

<p><strong>Electric.</strong> No electroreceptor has been identified in any crustacean, and none sought in
this species. Not a modelling gap; the state of the field. The physics is unambiguous: prey
bioelectric fields measured at microvolt scale with the electrode under a millimetre from
tissue, and the authors state the voltage from invertebrates was too weak to record away from
the source.</p>

<aside class="ui-source" id="ref-bedore2013">
  <a class="ui-source__link" href="https://doi.org/10.1086/669973" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Bioelectric Fields of Marine Organisms: Voltage and Frequency Contributions to Detectability by Electroreceptive Predators</span>
      <span class="ui-source__meta">
        Bedore et al.
        · 2013 · Physiological and Biochemical Zoology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>A behavioural sensitivity figure exists for a freshwater crayfish — a surrogate, different
order, fresh water.</p>

<aside class="ui-source" id="ref-patullo2010">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.039073" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Making sense of electrical sense in crayfish</span>
      <span class="ui-source__meta">
        Patullo et al.
        · 2010 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>The tool quotes named surrogates and will not produce a crab number.</p>

<p><strong>Welfare, which is a different question from detection.</strong> This species has nociceptors.
Acetic acid on every soft tissue tested — eyes, antennae, antennules, claws, leg joints —
produced a central nervous response, longer-lasting and lower in amplitude than a touch.</p>

<aside class="ui-source" id="ref-kasiouras2024">
  <a class="ui-source__link" href="https://doi.org/10.3390/biology13110851" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Putative Nociceptive Responses in a Decapod Crustacean: The Shore Crab (Carcinus maenas)</span>
      <span class="ui-source__meta">
        Kasiouras et al.
        · 2024 · Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>And green crabs <strong>learn to avoid a place where they are shocked.</strong> Given two shelters, with a
10 V, 180 Hz, 200 ms shock delivered every 5 s through wires on the legs in one of them, they
learned to walk left or right to reach the other. The voltage was set below the level at
which a single shock made a crab drop a leg, and some dropped a wired leg anyway.</p>

<aside class="ui-source" id="ref-magee2013">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.072041" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Shock avoidance by discrimination learning in the shore crab (Carcinus maenas) is consistent with a key criterion for pain</span>
      <span class="ui-source__meta">
        Magee et al.
        · 2013 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>Both read in full. That shock was contact current through the legs, not a field in water, so
it gives the tool <strong>no field threshold</strong> and changes no number above. What it changes is the
expectation: current is aversive to this animal, so an electric lure should be expected to
repel as well as attract. The welfare limit the tool enforces — crayfish forced electrotaxis,
about 4 V/m — marks where current <em>forces</em> movement, not where it becomes unpleasant.</p>

<p><strong>Magnetic.</strong> One directly relevant result: juvenile green crabs exposed to static magnetic
fields at strengths relevant to submarine power cables, <strong>females spending substantially more
time in exposed zones while males showed no consistent preference.</strong></p>

<aside class="ui-source" id="ref-james2025">
  <a class="ui-source__link" href="https://doi.org/10.1021/acs.estlett.5c00862" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Female Crabs Are More Sensitive to Environmentally Relevant Electromagnetic Fields from Submarine Power Cables</span>
      <span class="ui-source__meta">
        James et al.
        · 2025 · Environmental Science &amp; Technology Letters
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>

<p>A real, sex-specific response in this species — and a static-field spatial preference, not a
compass, and not a receptor. Nobody has located the transducer.</p>

<p><strong>The obvious confound, stated plainly.</strong> Helmholtz coils dissipate heat and crabs are
thermotactic. Working the published coil geometry through a thermal model gives, at the
strongest field over the exposure period, roughly <strong>20 W dissipated, a 0.58 K gradient across
the tank and a 0.30 K bulk rise</strong> — small, but not obviously below what an animal can detect,
and no behavioural thermal-discrimination threshold for this species could be found to
compare against. The model returns a number and refuses a verdict.</p>

<p>One weak argument against the thermal explanation: ohmic heating scales with the square of
the current, so the confound is about ten times larger at the strongest field than at the
intermediate one — while the reported attraction was <em>strongest at the intermediate field</em>.
Confound and effect run in opposite directions. <strong>A thermocouple in the tank would settle it,
and that is the cheapest experiment anywhere in this review.</strong></p>

<p>The usual comparison is the spiny lobster, the standard invertebrate magnetoreception system.</p>

<aside class="ui-source" id="ref-lohmann1984">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.113.1.29" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Magnetic Remanence in the Western Atlantic Spiny Lobster, Panulirus Argus</span>
      <span class="ui-source__meta">
        Lohmann
        · 1984 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-boles2003">
  <a class="ui-source__link" href="https://doi.org/10.1038/nature01226" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">True navigation and magnetic maps in spiny lobsters</span>
      <span class="ui-source__meta">
        Boles et al.
        · 2003 · Nature
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-ernst2016">
  <a class="ui-source__link" href="https://doi.org/10.1242/jeb.136036" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Effect of magnetic pulses on Caribbean spiny lobsters: implications for magnetoreception</span>
      <span class="ui-source__meta">
        Ernst et al.
        · 2016 · Journal of Experimental Biology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Here the abstract-only rule bites hardest:</strong> all three read at abstract, so their results
are not characterised. What can be said is about the shape of the literature rather than its
contents — the receptor cells have not been located and characterised in that animal either.
Mapping a mechanism from one order of crustaceans onto another, across more than two hundred
million years of divergence, when the source species’ anatomy is itself unresolved, produces
a hypothesis wearing borrowed credibility. The tool returns unavailable and says why.</p>

<h2 id="how-the-native-crabs-compare">How the native crabs compare</h2>

<p>The most informative part, because <strong>the comparison cannot be run.</strong></p>

<p>Across eight receptor channels and five species, green crab has measured values in five
channels and a described-but-unmeasured organ in two. For Dungeness, red rock, graceful rock
and yellow shore crab: <strong>two</strong> measured thresholds, both in Dungeness — a behavioural
detection threshold for a prey extract, and behavioural salinity detection measured by
antennular flicking.</p>

<aside class="ui-source" id="ref-pearson1979">
  <a class="ui-source__link" href="https://doi.org/10.1016/0022-0981(79)90005-4" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Thresholds for detection and feeding behavior in the dungeness crab, Cancer magister (Dana)</span>
      <span class="ui-source__meta">
        Pearson et al.
        · 1979 · Journal of Experimental Marine Biology and Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-sugarman1983">
  <a class="ui-source__link" href="https://doi.org/10.2307/1351397" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Salinity Detection and Associated Behavior in the Dungeness Crab, Cancer magister</span>
      <span class="ui-source__meta">
        Sugarman et al.
        · 1983 · Estuaries
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Both at abstract only, so those are descriptions of what was measured, not of what was
found</strong> — the model carries them with the same tag. (A third record sits off the matrix
entirely: dactyl chemo- and mechanoreceptor recordings in the kelp crab, not among the five.)</p>

<p><strong>Two filled cells out of thirty-two, and the comparison still cannot be run</strong> — for a
smaller reason than an empty literature. Those are <em>behavioural</em> thresholds, in grams per
litre and parts per thousand. Every green crab value is <em>single-unit electrophysiology</em>, in
micrometres or molar. Not the same quantity, so one row would be a category error rather than
a comparison.</p>

<p><strong>That is the state of the literature, not a gap in the modelling.</strong> Green crab is a classic
laboratory animal; the natives are commercially and ecologically important animals whose
sensory physiology has largely not been measured.</p>

<p>What <em>can</em> be compared is everything except the senses, and there the differences are
substantial and documented: salinity tolerance, depth and zonation, body size, moult timing,
tolerance of emersion and hypoxia.</p>

<aside class="ui-source" id="ref-young2019">
  <a class="ui-source__link" href="https://doi.org/10.3390/fishes5010004" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Life History and Population Dynamics of Green Crabs (Carcinus maenas)</span>
      <span class="ui-source__meta">
        Young et al.
        · 2019 · Fishes
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
  <p class="ui-source__ft"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M128 24a104 104 0 1 0 104 104A104.1 104.1 0 0 0 128 24Zm45.7 85.7-56 56a8 8 0 0 1-11.4 0l-24-24a8 8 0 0 1 11.4-11.4L112 148.7l50.3-50.4a8 8 0 0 1 11.4 11.4Z" /></svg> read at full text</p>
</aside>
<aside class="ui-source" id="ref-holsman2006">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps308183" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Intertidal migration and habitat use by subadult Dungeness crab Cancer magister in a NE Pacific estuary</span>
      <span class="ui-source__meta">
        Holsman et al.
        · 2006 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-defur1983">
  <a class="ui-source__link" href="https://doi.org/10.2307/1541467" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">ANALYSIS OF HEMOLYMPH OXYGEN LEVELS AND ACID-BASE STATUS DURING EMERSION 'IN SITU' IN THE RED ROCK CRAB, CANCER PRODUCTUS</span>
      <span class="ui-source__meta">
        DEFUR et al.
        · 1983 · The Biological Bulletin
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-moksnes2003">
  <a class="ui-source__link" href="https://doi.org/10.3354/meps250215" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Settlement behavior in shore crabs Carcinus maenas: why do postlarvae emigrate from nursery habitats?</span>
      <span class="ui-source__meta">
        Moksnes et al.
        · 2003 · Marine Ecology Progress Series
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-nicol2025">
  <a class="ui-source__link" href="https://doi.org/10.1111/maec.70071" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Comparison of Predatory Capabilities of Invasive European Green Crabs ( Carcinus maenas ) and Native Red Rock Crabs ( Cancer productus ) Preying Upon a Common Native Bivalve ( Leukoma staminea )</span>
      <span class="ui-source__meta">
        Nicol et al.
        · 2025 · Marine Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-jeppesen2024">
  <a class="ui-source__link" href="https://doi.org/10.1007/s10530-024-03467-3" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Recovering population of the southern sea otter suppresses a global marine invader</span>
      <span class="ui-source__meta">
        Jeppesen et al.
        · 2024 · Biological Invasions
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>The first was read at full text and the rest at abstract, which is why this section names
questions rather than answers.</p>

<h2 id="the-genetics-and-what-is-actually-there">The genetics, and what is actually there</h2>

<p>Looking for a genetic basis for the reproductive advantage — some identified difference
explaining why it out-reproduces the natives. <strong>There isn’t one, and the absence is
informative.</strong></p>

<p>The adaptive-genomics literature for this species is real and substantial. What it is <em>about</em>
is temperature: cold tolerance, thermal adaptation, a chromosomal inversion, and the
relationship between genotype and thermal plasticity.</p>

<aside class="ui-source" id="ref-tepolt2020">
  <a class="ui-source__link" href="https://doi.org/10.3389/fevo.2020.580701" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Rapid Adaptation to Temperature via a Potential Genomic Island of Divergence in the Invasive Green Crab, Carcinus maenas</span>
      <span class="ui-source__meta">
        Tepolt et al.
        · 2020 · Frontiers in Ecology and Evolution
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-thia2021">
  <a class="ui-source__link" href="https://doi.org/10.1111/mec.16258" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Ready on arrival: Standing variation at a chromosomal inversion contributes to rapid adaptation in an invasive marine crab</span>
      <span class="ui-source__meta">
        Thia
        · 2021 · Molecular Ecology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-venkataraman2025">
  <a class="ui-source__link" href="https://doi.org/10.1101/2025.04.22.650023" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Plasticity, not genetics, shapes individual responses to thermal stress in non-native populations of the European green crab ( Carcinus maenas )</span>
      <span class="ui-source__meta">
        Venkataraman et al.
        · 2025
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>Read at abstract only, so their findings are not characterised. But that the surveyed
literature concerns thermal physiology and not reproduction or sensory biology is an
observation about the literature, and it can be made.</p>

<p>So the honest account of why green crab out-reproduce the natives is life-history and
tolerance, not a gene: longer breeding season, earlier maturity at smaller size, two broods a
year where conditions allow, and sperm storage such that one fertilisation can serve more
than one clutch. Note that <em>reproducing</em> more is not the same as <em>mating</em> more — with sperm
storage the two can move in opposite directions.</p>

<h2 id="what-the-tool-is-for">What the tool is for</h2>

<p>The most-used outputs are refusals: no electric readout, no magnetic readout, no mixture
readout, no cross-species comparison, no sex difference in transduction. Sex enters in one
place — body size — because no measured threshold in this species differs by sex, and the
tool will not invent one.</p>

<p>The value is not in the numbers. It is that they cannot drift: every constant is pinned by a
test that fails if the figure is misquoted, and in one session those tests caught four errors
that had entered from secondary summaries of paywalled sources — which is how this literature
is normally read.</p>

<p><strong>The most instructive failure was mine, not the literature’s.</strong> The claim that no native
species had a single measured sensory channel was a strong negative drawn from a shallow
search, and it was wrong; a deeper search turned up the two Dungeness thresholds immediately.
<strong>A test had been pinning the wrong number in place</strong>, with a comment beside it admitting the
value was stale. That is worse than an unchecked number, because it looks checked.</p>

<p>Correcting it nearly introduced a new error. The function answering <em>which channels are
comparable across species</em> tested only whether a cell was marked measured. Filling the two
Dungeness cells would have made two channels report comparable when the underlying quantities
are not the same thing. It compares units now. <strong>A test that counts statuses will happily
certify a category error</strong>, and the correction is what exposed it.</p>

<p><strong>What would make it wrong:</strong> a measured audiogram for <em>Carcinus maenas</em>, Dungeness and red
rock crab on one rig, showing receptor bands substantially different from the surrogate
values used here. Most mechanical conclusions would need redoing. That measurement does not
exist, and it is the single experiment that would change the most.</p>

<h2 id="corrections">Corrections</h2>

<p><strong>2026-09-06.</strong> Three changes, none erasing anything above.</p>

<ul>
  <li>The native-comparison section originally said <em>“two measured chemosensory thresholds in a
single species and nothing else.”</em> The two are now cited by key, one is a salinity threshold
rather than a prey-odour one, and <strong>“nothing else” was an overreach</strong> — a third native
record exists off the matrix. Both are held at abstract only, so the post names what they
measured and not what they measured it to be. The count of filled cells is unchanged at two
of thirty-two, and the comparison remains un-runnable.</li>
  <li><strong>“What the tool is for”</strong> gains the account of how that error survived a test, and of the
second defect that correcting it exposed.</li>
  <li>The correction has been applied to the model itself, not only to this post.</li>
</ul>

<p><strong>2026-09-16.</strong> One addition, nothing erased: the electric section now carries the
green-crab welfare evidence — nociceptive responses and learned shock avoidance — with a
note that neither supplies a field threshold, so no number in the tool changed.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[A calculator that answers what a green crab can detect, in what units, at what range — and refuses to answer where nobody has measured. What it found about mechanoreception, chemistry, electric and magnetic fields, and how the native crabs compare.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/european-green-crab.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/european-green-crab.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry><entry><title type="html">“Frequencies” are just one piece of the puzzle</title><link href="https://polarize.tech/blog/what-a-wave-can-tell-you/" rel="alternate" type="text/html" title="“Frequencies” are just one piece of the puzzle" /><published>2026-09-01T11:00:00-06:00</published><updated>2026-09-01T11:00:00-06:00</updated><id>https://polarize.tech/blog/what-a-wave-can-tell-you</id><content type="html" xml:base="https://polarize.tech/blog/what-a-wave-can-tell-you/"><![CDATA[<p>Process note. Building a list of what a biological signal is known to carry, then pointing
the same reader at waves with nothing alive in them.</p>

<p>Starting observation: an ECG is not only a record of a heart contracting. Identity, sex, age
and health have all been read out of one. If that holds for a single signal, the question is
what <em>every</em> biological signal carries, and whether the same structural features carry it
each time.</p>

<h2 id="the-signals-catalogued">The signals catalogued</h2>

<p>Six, named by source tissue rather than application. Representative textbook ranges, not
hard bounds.</p>

<table>
  <thead>
    <tr>
      <th>signal</th>
      <th>source</th>
      <th>band</th>
      <th>amplitude</th>
      <th>shape</th>
    </tr>
  </thead>
  <tbody>
    <tr>
      <td><strong>ECG</strong></td>
      <td>myocardium</td>
      <td>~0.05–100 Hz</td>
      <td>1–10 mV</td>
      <td>strongly periodic, one sharp recurring event, consistent beat shape</td>
    </tr>
    <tr>
      <td><strong>EEG</strong></td>
      <td>cortex</td>
      <td>~0.5–100 Hz</td>
      <td>2 µV – 0.1 mV</td>
      <td>broadband, oscillatory, band-structured, weakly event-locked</td>
    </tr>
    <tr>
      <td><strong>EMG</strong></td>
      <td>skeletal muscle</td>
      <td>~2–500 Hz</td>
      <td>50 µV – 5 mV</td>
      <td>burst-structured, high-frequency, amplitude tracks effort</td>
    </tr>
    <tr>
      <td><strong>EOG</strong></td>
      <td>corneo-retinal dipole</td>
      <td>~DC–10 Hz</td>
      <td>10 µV – 5 mV</td>
      <td>slow steps and ramps; essentially DC</td>
    </tr>
    <tr>
      <td><strong>EDA</strong></td>
      <td>sweat glands</td>
      <td>~DC–2 Hz</td>
      <td>µS-scale</td>
      <td>slow level with responses on top; not oscillatory</td>
    </tr>
    <tr>
      <td><strong>EGG</strong></td>
      <td>stomach smooth muscle</td>
      <td>~0.03–0.15 Hz</td>
      <td>10–500 µV</td>
      <td>very-low-frequency near-sinusoidal pacemaker rhythm</td>
    </tr>
  </tbody>
</table>

<p><strong>The useful part was unexpected.</strong> Laid out together, the six separate on properties that
have nothing to do with physiology: how periodic, how sharp the events, where the spectral
weight sits, how much DC. You can tell them apart without knowing the tissue.</p>

<p>That is either an interesting fact about biological signals or an artefact of how they are
all recorded. Which one is not known here.</p>

<h2 id="the-information-axes">The information axes</h2>

<p>What kind of information is a biological wave known to carry. Each row is an entry point to
a literature.</p>

<p><strong>Identity.</strong> Attributing a trace to a specific person is a mature field for ECG, with a
parallel line on individuating signatures in EEG.</p>

<aside class="ui-source" id="ref-fratini2015">
  <a class="ui-source__link" href="https://doi.org/10.1186/s12938-015-0072-y" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Individual identification via electrocardiogram analysis</span>
      <span class="ui-source__meta">
        Fratini et al.
        · 2015 · BioMedical Engineering OnLine
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>
<aside class="ui-source" id="ref-chan2018">
  <a class="ui-source__link" href="https://doi.org/10.3389/fninf.2018.00066" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Challenges and Future Perspectives on Electroencephalogram-Based Biometrics in Person Recognition</span>
      <span class="ui-source__meta">
        Chan et al.
        · 2018 · Frontiers in Neuroinformatics
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Sex and age.</strong> Both have been read from short clinical recordings.</p>

<aside class="ui-source" id="ref-attia2019">
  <a class="ui-source__link" href="https://doi.org/10.1161/CIRCEP.119.007284" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Age and Sex Estimation Using Artificial Intelligence From Standard 12-Lead ECGs</span>
      <span class="ui-source__meta">
        Attia et al.
        · 2019 · Circulation: Arrhythmia and Electrophysiology
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p>The <em>discrepancy</em> between an age estimated from the signal and a person’s actual age has
itself been studied as a marker.</p>

<aside class="ui-source" id="ref-lima2021">
  <a class="ui-source__link" href="https://doi.org/10.1038/s41467-021-25351-7" rel="noopener">
    <span class="ui-source__icon" aria-hidden="true"><svg class="ui-icon" viewBox="0 0 256 256" aria-hidden="true" focusable="false"><path d="M224 48h-64a32 32 0 0 0-32 32 32 32 0 0 0-32-32H32a8 8 0 0 0-8 8v128a8 8 0 0 0 8 8h64a16 16 0 0 1 16 16 8 8 0 0 0 16 0 16 16 0 0 1 16-16h64a8 8 0 0 0 8-8V56a8 8 0 0 0-8-8Zm-104 8v113.6a32 32 0 0 0-24-9.6H40V64h56a16 16 0 0 1 16 16Zm96 104h-56a32 32 0 0 0-24 9.6V80a16 16 0 0 1 16-16h56Z" /></svg></span>
    <span class="ui-source__text">
      <span class="ui-source__title">Deep neural network-estimated electrocardiographic age as a mortality predictor</span>
      <span class="ui-source__meta">
        Lima et al.
        · 2021 · Nature Communications
      </span>
    </span>
    <span class="ui-source__go" aria-hidden="true">↗</span>
  </a>
</aside>

<p><strong>Autonomic and affective state.</strong> Heart-rate variability is the standard non-invasive
window onto autonomic balance; electrodermal activity indexes a sympathetic pathway
directly.</p>

<p><strong>Intention.</strong> Muscle activity decodes motor intent; cortical activity carries potentials
preceding movement rather than following it.</p>

<p><strong>Health.</strong> The axis with the most literature behind it, and the only one this bench has
measured anything on.</p>

<p>None of those papers was read at full text. They are cited as entry points; what they exist
to study is stated, not what any of them found.</p>

<h2 id="the-reframing">The reframing</h2>

<p>Building the list changed what the project looked like.</p>

<p>It had been treated as signal processing — extracting a feature from a trace. Laid out
together the axes look like a <strong>taxonomy</strong> problem instead.</p>

<p>Identity, sex and age barely change. State and intention change minute to minute. Health
drifts. Those are not the same kind of quantity, and calling them all “information in the
signal” hides the most important distinction between them.</p>

<p>That came from making a table, not from running anything.</p>

<h2 id="waves-with-nothing-alive-in-them">Waves with nothing alive in them</h2>

<p>A reader that finds rich structure in biological signals has to be asked whether it finds
rich structure in everything. So the same reader gets pointed at waves with no organism in
them:</p>

<ul>
  <li><strong>Tide gauges</strong> — two stations, 61 days. A blind read recovered the principal lunar
semidiurnal period and separated the moon’s contribution from the weather’s.</li>
  <li><strong>Solar flux against cosmic-ray flux</strong> — 14.6 years. Recovered the known anticorrelation,
but only given the full cycle. That makes it a result about <em>how much data you need</em>.</li>
  <li><strong>Seismic, infrasound, ocean sound, geomagnetic field</strong> — recovered the secondary
microseism and the daily solar-quiet variation, blind.</li>
</ul>

<p>The standing rule on that log:</p>

<blockquote>
  <p>A high structure score on a signal with no organism in it is a caution about the
instrument, not a finding about nature.</p>
</blockquote>

<p><strong>Reading tides well is partly bad news.</strong> The structure being found might be a property of
the reader rather than of life. Two of those runs did embarrass the instrument — one exposed
silent bugs at low sample rates, another showed a standard statistical null invalid on
deterministic signals.</p>

<h2 id="sound-light-water">Sound, light, water</h2>

<p>Mapped, not tested.</p>

<p>The structural properties in question — how loud, how bright, how periodic, how consistent
the repeating unit, whether a slow rhythm modulates a fast one — have natural readings in
sound and in light. Loudness and timbre in acoustics; brightness and colour in optics;
amplitude and morphology in a bioelectric trace. Water gave the cleanest test so far because
a tide is well enough characterised that the reader had nowhere to hide.</p>

<p>A correspondence you can write down is not one you have shown. Applying these
characteristics across modalities is, until tested the way the cardiac work was, <strong>a
hypothesis carried by analogy.</strong></p>

<h2 id="what-would-make-this-wrong">What would make this wrong</h2>

<p>If the structural characteristics separating biological signals turn out to separate <em>any</em>
filtered time series equally well, then the shared-grammar idea is an artefact of everyone
using similar pipelines, and this survey describes the pipeline rather than life. That is a
live possibility, it is why the non-biological waves get read at all, and nothing here rules
it out.</p>]]></content><author><name>Joshua Anderton</name></author><summary type="html"><![CDATA[Building a list of every kind of information a biological signal is known to carry, and which structural feature of the wave carries it — then asking the same question of tides, seismic noise and the solar cycle.]]></summary><media:thumbnail xmlns:media="http://search.yahoo.com/mrss/" url="https://polarize.tech/assets/posts/sea-wave.jpg" /><media:content medium="image" url="https://polarize.tech/assets/posts/sea-wave.jpg" xmlns:media="http://search.yahoo.com/mrss/" /></entry></feed>